
1. INTRODUCTION
Indian agriculture remains heavily dependent on the monsoon and hence very vulnerable to climate change. Rising global temperatures have led to increasingly erratic precipitation patterns, very often heavy rains followed by long dry spells. Within a season, India sometimes experiences two extremes—flood and drought. Drought can cause significant reductions in yield for essential crops such as rice, and wheat leading to severe economic losses particularly impacting marginal farmers. Between 2016 and 2022, 33% crop loss was recorded due to drought in India [1]. For Indian farmers, particularly in Marathwada and Vidarbha regions of Maharashtra, who are already located in the rain-shadow zone of the Western Ghats, droughts pose a major challenge [2].
Water stress activates adaptive changes in plants, which help to decrease water loss, improve uptake of water by plant roots, and protect cell processes by increased production of reactive oxygen species (ROS) and osmolytes such as proline. Excessive drought stress leads to stunted plant growth as plants exhibit decreased growth and wilting, accompanied by limited photosynthesis due to closure of stomata [3]. Recent methods to tackle drought include the use of nanotechnology, drought-resistant crop varieties, absorbent materials, film farming, etc. An alternate strategy is the use of plant-growth-promoting bacteria (PGPB).
PGPB are a group of diverse soil bacteria that thrive in the soil around plant roots and positively impact the growth of plants. These bacteria aid in plant growth promotion by using a combination of different mechanisms. These include direct mechanisms like enhancing nutrient uptake and regulating phytohormones, and indirect mechanisms like controlling plant pathogens and increasing plant viability in stress conditions [4]. These bacteria help plants mitigate various abiotic stresses arising from changes in pH, temperature, or osmotic pressure, as well as exposure to ultraviolet (UV) radiation or oxidative stress, by inducing systemic tolerance. This tolerance involves multiple physical and biochemical processes within the plant [5]. Mechanisms proposed to explain how PGPB enhance drought tolerance include modification of root architecture, production of auxins, volatile organic compounds, 1-aminocyclopropane-1-carboxylic acid (ACC) deaminase, and exopolysaccharides (EPS) [3]. Owing to these beneficial effects, PGPB are widely exploited in agriculture through their application as biofertilizer formulations to enhance crop growth, making them an effective and eco-friendly alternative to harmful chemical fertilizers.
In the present study, the plant growth-promoting (PGP) potential of six soil bacterial isolates was evaluated, along with their ability to mitigate drought stress in wheat (Triticum durum L., variety Pusa Tejas HI 8759). This was assessed by analyzing parameters such as seed germination, plant morphological traits, chlorophyll content, antioxidant activity, and ROS accumulation in plants grown from isolate-inoculated wheat seeds under drought conditions. Of the six isolates, Kocuria turfanensis and Kocuria rosea demonstrated good drought tolerance and significantly enhanced wheat growth. Kocuria species have been previously reported to alleviate salt stress in maize and tomato [6,7]. This study is the first systematic demonstration of Kocuria spp. ameliorating drought stress specifically in T. durum. With wheat being a crucial, drought-sensitive staple, this finding has major implications for agricultural productivity, especially in India’s semi-arid regions.
2. MATERIALS AND METHODS
2.1. Soil Sampling and Isolation of Bacteria
Rhizosphere soil samples were collected in polyethylene zip-lock bags from crop fields located in Uttan (19.27884°N, 72.79905°E) and from the mangrove region of Vashi, Navi Mumbai, Maharashtra (19.0762° N, 72.9881° E), India. Soil samples were sieved through a mesh before bacterial screening. Soil samples (5 g each) were added to 100 ml sterile saline solution (0.85% NaCl) in a 250 ml Erlenmeyer flask. Flasks were kept at room temperature for a day with intermittent shaking. From this suspension, 100 μl was spread onto nutrient agar plates (HiMedia M001) and incubated at room temperature for 48 hours. The morphology and Gram nature of the isolates obtained were studied, and pigment production, if any, was noted (Supplementary Table 1). Each of the isolates was assessed for PGP characteristics. A few selected organisms were identified by biochemical tests and 16S rDNA sequencing (GenBank accession numbers - PZ623524, PZ623525)
2.2. Characterization of Bacterial Isolates
The isolates were tested for nitrogen-fixing ability by growing on Ashby’s agar plates (HiMedia M706) after 5 days of incubation at 25°C ± 2°C. The phosphate-solubilizing activity was determined using Pikovskaya’s agar and National Botanical Research Institute's Phosphate (NBRIP) agar [8,9] by spot inoculating the bacterial isolates to check zones of clearance around colonies as an indication of phosphate solubilization. Similarly, potassium solubilizing activities were checked on Aleksandrow’s medium (HiMedia M1996).
Production of siderophores was determined by a change in color, surrounding the bacterial colony in Chrome Azurol S (CAS) agar plate due to the removal of iron from CAS dye by the siderophores being produced as suggested [9]. A loopful of bacterial isolates was inoculated in peptone water base and kept under shaking conditions for 48–72 hours at 25°C ± 2°C, followed by the addition of Nessler’s reagent to form a yellow-brownish precipitate indicating ammonium production [9].
2.2.1. Production of indole acetic acid (IAA)
The production of IAA was determined both qualitatively and quantitatively using Salkowski’s reagent [10]. Twenty-four-hour-old bacterial cultures were inoculated in Nutrient Broth (HiMedia M002) enriched with 0.1% tryptophan and incubated at 25°C ± 2°C on a shaker for 5 days. For qualitative analysis, 2 ml Salkowski’s reagent was added to 1 ml of inoculated broth and incubated for 30 minutes in the dark to observe a color change from yellow to pink. For quantitative analysis, 1,000 μl of inoculated broth was transferred to sterile Eppendorf tube and centrifuged for 10 minutes at 10,000 rpm from which, 50 μl of the supernatant was added in a 96-well microtiter plate along with 100 μl Salkowski’s reagent, kept under dark conditions for 30 minutes, followed by estimating the absorbance of the pink color produced at 530 nm using Elisa Plate reader (SpectraMax®-iD3 Multi-mode Microplate Reader, USA). The concentration of IAA produced μg/ml by each isolate was estimated using the standard plot of IAA.
2.2.2. Investigation of drought tolerance
Resazurin microtiter assay (REMA) [11] was used to determine the viability of metabolically active cells. The exponential phase cultures of each isolate were inoculated in Trypticase Soy Broth containing polyethylene glycol (PEG)-6000 [12] at a concentration ranging between 10% to 40% and were incubated at 25°C ± 2°C with continuous agitation for 5 days. Following the incubation period, 100 μl of inoculated broth was incubated with Resazurin dye for 2 hours at 37°C in a sterile microtiter plate for its conversion to resorufin, whose fluorescence was determined at 535–585 nm using an ELISA Plate reader (SpectraMax®-iD3 Multi-mode Microplate Reader, USA).
2.2.3. Production of IAA under drought stress
The 24-hour-old cultures of bacterial isolates were inoculated in nutrient broth supplemented with 0.1% tryptophan and PEG-6000 and were incubated at 25°C ± 2°C, under shaking conditions for 5 days. The amount of IAA produced was determined spectrophotometrically at 530 nm using Salkowski’s method.
2.2.4. UV-resistance analysis
Each of the bacterial suspensions (OD600 = 0.1), 10 ml, was placed in a Petri plate base and exposed to UV for 10, 15, 20, 30, and 40 minutes, and the samples taken at each time interval were serially diluted 10-fold thrice. The cfu/ml of each bacterial isolate was estimated by the drop count method, which is a faster and more economical way of enumeration [13]. Drought-prone areas frequently experience intense solar radiation. Hence, PGPB strains that are both drought-tolerant and UV-resistant have a potential advantage. The tests were done in three technical replicates.
2.3. Seed Surface Sterilization and Germination
Wheat (Pusa Tejas HI 8759) seeds were soaked for 24 hours in clean tap water and rinsed 3–5 times. Subsequently, the seeds were treated with 0.1% HgCl2 for 1 minute [14], and washed 5 times with sterile water. The surface-sterilized seeds were then transferred to a sterile Petri plate with sterile filter paper and kept for germination at room temperature for 5–7 days. Sterile distilled water was added at regular intervals to maintain the optimum moisture content required for the germination of seeds.
2.4. Agar Butt Assay to Evaluate Plant Growth Promotion Under Osmotic Stress
The ability of the bacterial isolates to tolerate osmotic stress and promote plant growth was evaluated in-vitro using 2% agar butts with varying concentrations of PEG-6000 in 65 ml tubes. Surface-sterilized wheat seeds (three each) were added to five water agar butts pre-inoculated with 100 μl of exponential bacterial culture
(OD600 = 0.2) and were incubated at 25°C ± 2°C for 15-17 days under laboratory conditions with a 12 hours light/12 hours dark photoperiod, using two 40 W lamps. A concentration range of 10%–30% of PEG-6000 was employed. The uninoculated water agar butts served as controls. The assay was done in three replicates.
2.5. Pot Experiment to Evaluate Plant Growth Promotion Under Drought Stress
Germinated wheat seeds were grown in pots containing sterilized, oven-dried soil (80°C for 3–4 hours). Each test pot was filled with 150 g of soil inoculated with 10 ml of a 1:10 diluted bacterial culture (OD600 = 0.2) and sown with 10 germinated seeds, in triplicate. Two types of controls were set up and each type of control pot was filled with 150 g of soil inoculated with 10 ml of water (instead of culture) and sown with 10 germinated seeds, in triplicate. The first set of control pots were watered every day. This maintained soil moisture at 60%–70% field capacity throughout (CW, control-well watered). The other set of control pots were watered for 15 days every day and for the next 15 days were watered on alternate days. This decreased soil moisture to 20%–30% field capacity (CWW—alternate day watering). The test pots inoculated with culture were watered like the CWW to maintain drought-stressed conditions. Soil moisture was monitored regularly using a portable soil moisture meter. All the plants were grown for 30 days under a 12-hour photoperiod.
Gravimetric monitoring of soil moisture was also performed where soil samples were collected at weekly intervals, and moisture was determined by oven-drying at 105°C until constant weight. The water loss was calculated as the difference between the current weight and the target weight using the following formula:
Soil moisture (%) = (Fresh soil weight−Dry soil weight) × 100 /Dry soil weight
Plant health and growth parameters in bacteria-inoculated pots were compared with uninoculated control pots to assess PGP activity under drought stress. The pot experiment was conducted three times using three different soil samples. The soils used for the experiments contained moderate levels of organic carbon and phosphate, low to medium nitrate content, and moderate potassium levels, as determined by qualitative analysis.
2.6. Estimation of Plant Morphological Parameters
The plants that grew in the water agar butt assay and pot assay were uprooted and washed. Wet weight (g), shoot, and root length (cm), and width of leaves (μm) were determined for each plant [15]. Leaf width was measured using a microscope imaging software (Leica Application Suite × 3.7.5.24914, 2021, Leica Microsystems). Ten plants per treatment were used for each measurement.
2.7. Preparation of Acetone Extract of Leaves
Acetone (80%) was used to extract chlorophyll, flavonoids, and polyphenols from leaf samples (1.2 g) collected from both agar butt and pot experiments. The extraction procedure used by Li et al. [16] was modified to ensure consistent extraction efficiency. Leaf samples (1.2 g) were homogenized thoroughly using a mortar and pestle with 10 ml of 80% acetone. The resulting mixture was transferred into a 15 ml Falcon tube and centrifuged at 2,000 rpm for 10 minutes. The supernatant obtained was used for the estimation of biochemical parameters.
2.7.1. Estimation of chlorophyll content
Chlorophyll a is more abundant than chlorophyll b in plants. Therefore, chlorophyll a content was estimated following the protocol described earlier [16]. Briefly, 100 μl of the samples were taken, and the absorbance was determined at 663 nm spectrophotometrically in a microtiter plate using an ELISA Plate reader (SpectraMax®-iD3 Multi-mode Microplate Reader, USA). As the experimental objective focused on relative differences between treated and control groups rather than absolute quantification, raw absorbance values at 663 nm were utilized directly for comparative analysis.
2.7.2. Estimation of total polyphenols
The total polyphenolic content in leaf extracts was determined using 100 μl Folin–Ciocalteu reagent incubated with 20 μl sample for 10 minutes, followed by addition of 10 μl saturated sodium bicarbonate solution and subsequent incubation for 30 minutes at 25°C ± 2°C. The concentration of total polyphenols present in the leaf extract was determined using a tannic acid standard curveThe procedure was adapted from the methods reported earlier with some modifications [17,18].
2.7.3. Estimation of flavonoids
Total flavonoid content was checked using 100 μl of 2% AlCl3 incubated with 50 μl of the sample for 30 minutes at 25°C ± 2°C and taking absorbance at 420 nm spectrophotometrically in a microtiter plate using an ELISA Plate reader (SpectraMax®-iD3 Multi-mode Microplate Reader, USA) [19].
2.7.4. Determination of antioxidant activity by 1,1-diphenyl-2-picrylhydrazyl (DPPH) assay
The radical scavenging activity of the plant leaf extract was determined using 0.1 mM DPPH reagent according to the published protocol [20]. The sample (50 μl) was incubated with 150 μl of DPPH reagent under dark conditions for 30 minutes at 25°C ± 2°C. The percentage scavenging activity was calculated using the formula:
% Scavenging = (Absorbance of control - Absorbance of test sample) × 100/Absorbance of control
2.8. Estimation of ROS Accumulation
The amount of ROS accumulated in the plant cells was observed microscopically and analyzed using 2-7-Dichlorodihydrofluorescein diacetate (DCFDA) [21]. 10 mM DCFDA prepared in Dimethyl sulfoxide was used to stain root and leaf samples of both test and control plants, and samples treated with 0.5 mM H2O2 for 15 minutes served as a positive control. The leaf and root samples were stained with DCFDA for 15 minutes and washed with distilled water three times, blotted, and observed for fluorescence under the blue filter of a fluorescence microscope. Images were captured and derived from a microscope imaging software (Leica Microsystems).
2.9. Enumeration of Root-Associated Bacteria
Surface-sterilized wheat seeds were grown in water agar butts and pots pre-inoculated with a log-phase bacterial culture. The plants were harvested, and the soil loosely attached to roots (pot experiment) was removed by gentle shaking. The roots were cut and then aseptically transferred to 10 ml normal saline with 20 sterile glass beads, vortexed for 2–3 minutes to detach the surface-associated bacterial cells. The viability of bacteria colonizing the root surface was determined using the principle of REMA [22,23]. Briefly, 100 µl of that suspension is added to a well of a sterile black 96-well microtiter plate along with 50 μl of double strength nutrient broth and 30 μl of resazurin (0.015% v/v). The microtiter plate is incubated for 2 hours and then fluorescence is estimated at 540–585 nm excitation and emission wavelengths in a fluorescence plate reader (iD3 spectra drop, Molecular Devices). Similarly, the viable bacterial count was also determined using the Standard Plate Count method..
2.10. Soil Microbiome Analysis
Unlike previous pot experiments, unsterilized garden soil was used for the study. Each pot (150 g soil) was inoculated with 10 ml of a 1:10 diluted bacterial culture (OD600 = 0.2) and sown with 10 germinated wheat seeds, in triplicate. Plants were grown for 30 days under a 12-hour photoperiod, with daily watering for 15 days followed by alternate-day watering, and soil moisture was monitored regularly.
Soil samples were collected on the 30th day of the pot assay from the pots inoculated with the two selected isolates, uninoculated control pots with and without drought stress. The samples from replicate pots receiving the same treatment were pooled, thoroughly mixed and used for microbiome analysis. The raw sequence data obtained from the soil samples were stored in FASTQ files, and the sequence information or paired-end reads' quality was inspected using QIIME 2 [24]. While processing the reads, every run was denoized separately with same parameters, a 17-bp left trim and 21-bp right trim were used for primer removal, along with truncation to 270 and 210 bp for the forward and reverse reads, respectively, to remove low-quality bases at the end of the reads. After denoizing DADA2 clusters, amplicons, and outputs, amplicon sequence variants (or ASVs) were determined [25]. To determine taxonomy, QIIME 2 feature classifier function was used with Greengenes2 2022.10.backbone.full-length database trained for V3-V4 region. The average species diversity within a sample or a niche, along with diversity between the samples, was compared. Twenty taxonomic lineages were found, and those not included in the top 20 were collapsed as “Others”, while the ones that had not been classified had been collapsed under the category of “unclassified”. The metagenomic sequencing data have been submitted to the NCBI Sequence Read Archive with an accession number PRJNA1489532.
2.11. Statistics
For data analyses, statistics software SigmaStat 3.5 was used. Standard errors and means for a minimum of three replicates were used to calculate each parameter. Student's t-test or one-way ANOVA and a post hoc test (Tukey's test) (* ~ p < 0.05) was used to analyze the data obtained from different experiments. The differences between the control and treatment groups were examined.
3. RESULTS
3.1. Bacterial Isolates and Their PGP Characteristics
Six isolates were selected, viz., CMG-1, MAN, FS-1, ANK-6, KPC, and KAD. These were tested for individual PGP characteristics (Supplementary Table 1). KPC and KAD formed pink and orange-red colonies, respectively, suggesting carotenoid production. These cultures were grown in broth, and the cells were pelleted, and methanol was added to the pellet. The maximum absorbance of the methanol extracts was determined to be 471 nm for KPC and 450 nm for KAD. These values fall within the characteristic range for carotenoids, which absorb light typically between 450 and 500 nm. The isolate KPC has been previously identified in our lab, and its pigment has been studied in greater detail [26].
3.2. Production of IAA
The amount of IAA produced by bacteria was determined using Salkowski’s reagent. All isolates produced IAA, with KPC giving the highest concentration of 60.67 μg/ml under normal growth conditions in Nutrient broth after 5 days. Under osmotic stress (induced by growing the bacterial cells with PEG-6000 in Nutrient broth with 0.1% tryptophan), the production of IAA by each isolate was seen to decline with increasing concentration of PEG-6000. Four isolates, KPC, KAD, MAN, and CMG-1, showed IAA production (5.7–7.3 μg/ml) even at 40% PEG-6000 (Fig. 1).
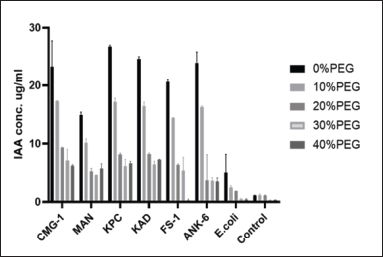 | Figure 1. Production of IAA by bacterial isolates in nutrient broth with 0.1% tryptophan in the presence of PEG-6000 was determined spectrophotometrically at 530 nm using Salkowski’s method. [Click here to view] |
3.3. Drought Tolerance and UV Resistance
The effect of PEG-6000 on bacterial growth and viability was determined using resazurin viability assay or REMA (Fig. 2A). When exposed to osmotic stress conditions in the presence of PEG-6000, the isolates CMG-1, KPC, KAD, MAN, ANK-6, and FS-1 displayed were able to tolerate 30% of PEG-6000 but the viability of the MAN strain reduced in the presence of 30%–40% PEG-6000 (Fig. 2A). Though the isolates, ANK-6 and FS-1 grew well in 30% PEG-6000 their IAA production was markedly low (Fig. 1).
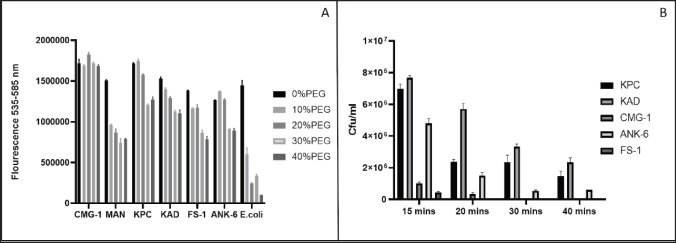 | Figure 2. A) Viability of bacterial isolates grown in the presence of PEG-6000 assessed by the Resazurin assay. B) Assessment of UV tolerance in selected osmotic stress-tolerant bacterial isolates using the drop count method. [Click here to view] |
The bacterial isolates that tolerated osmotic stress, viz., CMG-1, KPC, KAD, ANK-6, and FS-1, were further subjected to increasing durations of UV exposure (Fig. 2B). UV tolerance of these isolates was assessed using a viable drop count assay and expressed as cfu/ml following 15, 20, 30, and 40 minutes of exposure. After 15 minutes, KAD and KPC demonstrated the highest survival, with viable counts of approximately 7–8 × 10⁶ and 6–7 × 10⁶ cfu/ml, respectively. ANK-6 showed moderate tolerance (4–5 × 10⁶ cfu/ml), whereas CMG-1 and FS-1 exhibited substantially lower viable counts, indicating greater sensitivity to UV radiation.
With prolonged exposure, a progressive decline in viability was observed across all isolates. By 40 minutes, only KPC and KAD retained appreciable viability, ANK-6 showed poor survival, and CMG-1 and FS-1 displayed near-complete loss of viability. Notably, KPC and KAD also exhibited enhanced pigment production following UV exposure, suggesting a possible protective response to UV-induced stress.
3.4. Agar Butt and Pot Experiment to Evaluate Plant Growth Promotion Under Stress Conditions
Five isolates, viz., KPC, KAD, CMG-1, ANK-6, and FS-1, were used for agar butt assay (0%–30% PEG- 6000) and Pot assay with selected wheat cultivar Pusa Tejas HI 8759. In the agar butt assay, wheat plants were harvested after 15 days and assessed for key morphological parameters. Although plants grown in the presence of KPC and KAD showed an overall improvement in growth compared to controls, the differences were not statistically significant under agar-based conditions (results not shown). On the contrary, soil pot experiments revealed a clear and significant enhancement of plant growth in response to KPC and KAD inoculation (Fig. 3). Plants were harvested after 30 days, and those treated with KPC and KAD exhibited significant increases (p < 0.05) in individual root length, fresh biomass, and leaf width compared to the untreated control with alternate-day watering (CWW) (Fig. 3; Supplementary Fig. 1). Statistical analysis was performed using pot means from three independent experiments, each conducted with three sets of 10 plants. The lack of statistically significant growth in agar butts may be because the conditions do not replicate soil-like conditions.
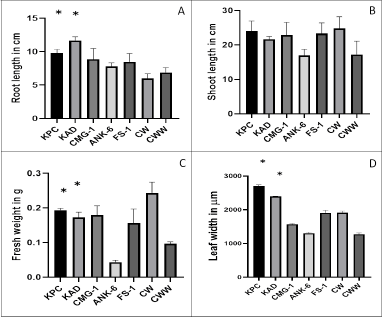 | Figure 3. Growth-promoting effects of bacterial isolates on wheat plants under water-deficit conditions. Wheat plants were inoculated with KPC, KAD (Kocuria spp.), CMG-1, ANK-6, or FS-1 and evaluated for (A) root length (cm), (B) shoot length (cm), (C) fresh weight (g), and (D) leaf width (μm). Well-watered uninoculated plants (CW) and uninoculated plants subjected to alternate-day watering (CWW) were included as controls. Values are presented as mean ± SD (n = 3). Asterisks (*) denote statistically significant differences (p < 0.05) relative to the alternate-day watered uninoculated control (CWW). [Click here to view] |
3.5. Comparison of the Five Isolates Across Multiple Parameters
Of the five isolates, KPC, KAD, CMG-1, ANK-6, and FS-1, only KPC and KAD maintained multiple PGP functions such as IAA production, viability, and plant growth promotion under combined osmotic, UV, and drought stress. CMG-1 showed sensitivity to UV but maintained reasonable performance with respect to viability and IAA production under osmotic stress and plant growth promotion under drought stress. ANK-6 and FS-1 were moderately viable and produced some IAA at high PEG concentrations but showed marked sensitivity to UV exposure. Both promoted limited plant growth under drought stress. On the other hand, MAN produced IAA under osmotic stress but could not promote plant growth under drought conditions.
Two of the five isolates, KPC and KAD, were found to be carotenoid producers, and it was observed that exposure to UV increased pigment production. The correlation between UV resistance and drought tolerance among isolates (highest in KPC and KAD) suggests that pigment production may be responsible for this. Table 1 summarizes how the isolates compare across multiple parameters. It can be clearly observed that both KPC and KAD demonstrate robust PGP traits under drought conditions (Table 1).
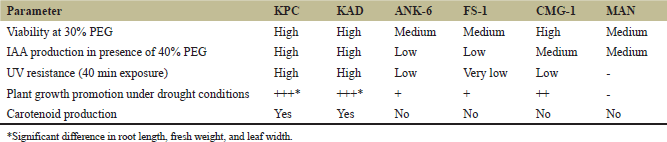 | Table 1. Comparison of KPC, KAD, ANK-6, FS-1, CMG-1, and MAN across multiple parameters. [Click here to view] |
Based on 16S rRNA gene sequencing and phylogenetic analysis, the isolates KPC, KAD, ANK-6, and FS-1 were identified as Kocuria turfanensis, Kocuria rosea, Acinetobacter junii, and Klebsiella aerogenes, respectively. CMG-1 was tentatively identified as Azotobacter sp. based on morphological, cultural, and biochemical characteristics.
3.6. Plant Chlorophyll Content, Antioxidant Content, and ROS Accumulation
Wheat plants inoculated with K. turfanensis and K. rosea showed a significant increase (p < 0.05; n = 3) in chlorophyll content compared to untreated drought-stressed controls (Fig. 4A). There was maximum increase in chlorophyll content (more than two-fold higher) in plants inoculated with K. turfanensis and K. rosea as compared to other isolates (1.2–1.4-fold). Enhanced chlorophyll levels indicate improved photosynthetic capacity under water-limiting conditions.
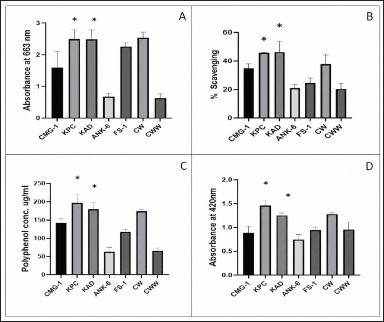 | Figure 4. Influence of bacterial strains on chlorophyll content and antioxidant responses of plants under drought stress. (A) Chlorophyll content measured at 663 nm (B) Antioxidant activity expressed as percentage DPPH radical scavenging (C) Total polyphenol content (μg TAE/g) and (D) Total flavonoid content. Plants inoculated with K. turfanensis (KPC) and K. rosea (KAD) showed significantly higher chlorophyll levels and antioxidant capacity compared to untreated drought-stressed controls. Controls: CW -Well-watered uninoculated plants; CWW—uninoculated plants subjected to alternate-day watering. Asterisks (*) denote statistically significant differences (considering three sets of independent experiments, p < 0.05). [Click here to view] |
A marked increase in antioxidant defense was observed in plants treated with Kocuria spp., reflecting a protective response against drought-induced oxidative stress. Quantitative antioxidant analysis using the DPPH radical scavenging assay revealed a significant elevation in ROS scavenging activity (p < 0.05; n = 3) in Kocuria-inoculated plants (Fig. 4B). Under drought stress, plants treated with K. turfanensis and K. rosea exhibited substantially higher scavenging activities in their leaf extracts (45.75% and 46.34%, respectively) compared to control plants (20.45%). Plants treated with other isolates showed much lower scavenging activity.
Total polyphenol (Fig. 4C) and flavonoid contents (Fig. 4D), which play key roles in cellular redox homeostasis, were also significantly higher only in Kocuria-treated plants. Polyphenol content was 2.7-2.9-fold higher, and flavonoid content was 1.2–1.5-fold higher compared to CWW.
Although the DPPH, total polyphenol, and flavonoid assays provide measures of overall antioxidant potential and phenolic compound accumulation, they do not directly assess enzymatic antioxidant activities (e.g., superoxide dismutase, catalase, and peroxidase) or redox-active metabolites (e.g., ascorbate and glutathione).
The enhanced antioxidant status correlated with reduced intracellular ROS accumulation, as confirmed by DCFDA staining. Roots of plants inoculated with Kocuria spp. displayed markedly lower ROS fluorescence compared to untreated controls, indicating efficient mitigation of oxidative stress under drought conditions (Fig. 5).
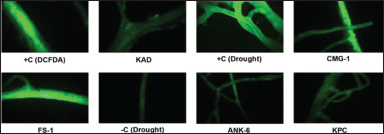 | Figure 5. ROS accumulation in the root region of plants grown in drought conditions. There was a markedly lower ROS fluorescence in the root region of plants inoculated with Kocuria sp. [Click here to view] |
3.7. Enumeration of Root-Associated Bacteria from Pot Assay
To confirm that the inoculated bacteria formed an association with the plant root surfaces, the number of viable bacterial cells on the root surfaces of pot-grown plants was determined using the Resazurin viability assay [22] and the viable count assay. It was then found that there was an increase in the number of bacteria associated with plant roots as compared to the uninoculated control. The increase was maximum for K. rosea (KAD, 3.6 × 10⁶ cfu/ml), followed by K turfanensis (KPC, 2.2 × 10⁶ cfu/ml), Acinetobacter junii (ANK-6, 1.9 × 10⁶ cfu/ml), Klebsiella aerogenes (FS-1, 1.6 × 10⁶ cfu/ml), Azotobacter sp (CMG-1, 2 × 10⁶ cfu/ml .The comparatively higher counts of Kocuria strains suggests their greater persistence in the root-associated region (Fig. 6).
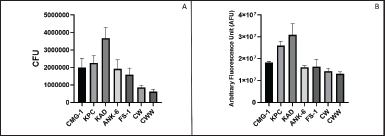 | Figure 6. Root-associated bacterial populations (pot assay) were measured by two independent methods: (A) Colony-forming units (CFU) recovered from wheat roots after inoculation with the five isolates for 30 days and control treatments. (B) Fluorescence intensity (measured in arbitrary fluorescence units, AFU) was determined using a resazurin-based fluorescence assay, which estimates bacterial metabolic activity on the root surface, which correlates with bacterial viability and presence. Controls: CW -Well-watered uninoculated plants; CWW—uninoculated plants subjected to alternate-day watering. [Click here to view] |
These methods provide strong evidence for root-associated bacterial populations but do not resolve spatial distribution. The presence of inoculated bacteria in the root region may contribute to the alteration of root morphology and thus enhance plant growth under drought conditions.
3.8. Microbiome Analysis of Soil
Considering the exceptional performance of Kocuria strains under osmotic, UV, and drought stress, soil microbiome analysis was carried out using the two Kocuria isolates.
A total of 4476 ASVs (amplicon sequence variants) were detected after appropriate filtering and the removal of archaea features from four soil samples, namely: CW, an uninoculated control soil with normal watering; CWW, an uninoculated control sample with alternate-day watering; KPC, soil inoculated with K. turfanensis; and KAD, soil inoculated with K. rosea. The mean length of all the sequences was 410 bp. Two ASVs (features) were detected for Kocuria sp., one in each inoculated sample. These ASVs were absent in the CWW and CW control samples. The length of the KPC ASV sequence was 408 bp, while that of KAD was 407 bp. The raw abundance of Kocuria spp. in KPC and KAD samples was 0.05% and 0.03%, respectively (Fig. 7A and B). Preliminary observations appear to show a shift in the abundance of phylum and class Actinobacteria, and families Micrococcaceae, Beijerinckiaceae, Azospirillaceae, Myxococcaceae, Geminicoccaceae, and Burkholderiaceae in the KPC and KAD treated samples. These shifts may reflect sampling variability rather than true treatment effects, as the results are based on single samples and, therefore, it is not possible to draw any definitive ecological conclusions. To determine whether Kocuria inoculation produces soil microbiome changes will require future studies to have adequate replication, deeper sequencing coverage, and functional metagenomic analyses.
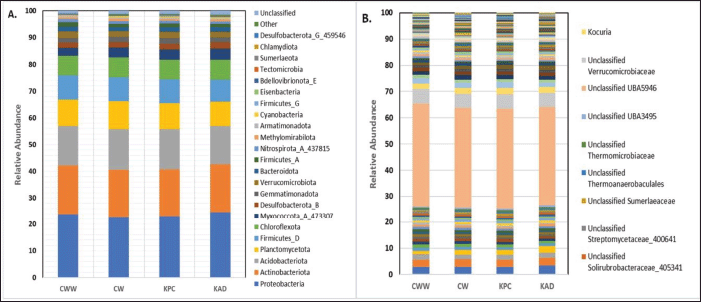 | Figure 7. A and B indicates the relative abundance (%) of bacterial phyla and genus, respectively, in treated and untreated soil samples. CW uninoculated control soil with normal watering, CWW uninoculated control sample with alternate-day watering, KPC soil with K. turfanensis with intermittent watering, and KAD soil with K. rosea with intermittent watering. [Click here to view] |
4. DISCUSSION
The present study explored the potential of soil-derived bacteria to mitigate drought stress in wheat. All six isolates, KPC, KAD, CMG-1, MAN, ANK-6, and FS-1, screened exhibited multiple PGP traits, including nitrogen fixation, phosphate and potassium solubilization, and production of IAA and siderophores. ANK-6 (A. junii) and FS-1 (K. aerogenes) produced minimal IAA under osmotic stress and showed marked sensitivity to UV exposure. ANK-6 and FS-1, thus, may be suitable for plant growth promotion under normal soil conditions. KPC, KAD, CMG-1, and MAN, in contrast, produced IAA even under severe osmotic stress (40% PEG-6000), indicating adaptation of these organisms to water-limiting conditions. Maintenance of IAA levels, albeit decreased, by these bacteria makes them good potential bioinoculants as they can be expected to function effectively even under environmental stresses. Of these, three isolates—KPC (K. turfanensis), KAD (K. rosea), and CMG-1 (Azotobacter sp.)—not only retained the ability to produce IAA but also promoted plant growth under drought stress.
Many Azotobacter species produce copious amounts of EPS, most commonly alginate [27]. EPS increases the soil’s water-holding capacity, entraps nutrients for plant growth, and encourages biofilm formation. This promotes plant growth under drought conditions [28]. The Azotobacter isolate (CMG-1) in this study also produced EPS, which may be responsible for its drought tolerance. CMG-1 did not produce any dark pigment; Azotobacter are known to produce the water-soluble pigment, melanin, which can absorb UV radiation, contributing to UV resistance of many bacteria. Absence of melanin could be the reason why CMG-1 was sensitive to UV [29,30]. This isolate, therefore, could only be useful in low-UV environments such as hydroponics or greenhouses.
Wheat plants inoculated with the Kocuria strains showed significant increases in root length (cm), fresh weight (g), and leaf width (µm) (p < 0.05) under drought stress as compared to controls. IAA regulates root architecture, lateral root formation, and root hair development, which are crucial for water uptake [31]. The sustained IAA production by Kocuria spp under osmotic stress is probably the reason for the significant increase in root length of wheat plants. Enhanced root development is crucial for drought tolerance, as deeper and more extensive root systems enable plants to access water from greater volumes and depths. Absence of significant differences in shoot length may indicate plants giving precedence to root growth over shoot growth so as to maximize water acquisition under drought stress. PGPB are known to trigger the accumulation of proline, glycine, betaine, etc. in plants under water stress [32]. The higher biomass is suggestive of Kocuria inducing plants to accumulate osmolytes, which is typically observed in plants under drought stress.
Chlorophyll content, polyphenol content, and flavonoid levels were also significantly higher in wheat plants treated with K. turfanensis and K. rosea. Chlorophyll content has been reported to decrease when the water content of the soil goes down. If plants maintain higher chlorophyll levels when there is a water deficit, they will be able to use light efficiently and therefore resist drought to a great extent [33]. The more than two-fold increase in chlorophyll content of Kocuria inoculated plants may, thus, enable plants to maintain photosynthetic capacity.
Our data showed that in Kocuria inoculated plants, there was higher DPPH radical scavenging activity, 2.7-2.9-fold higher polyphenol accumulation, 1.2–1.5-fold higher flavonoid content and markedly reduced ROS in roots. Polyphenols and flavonoids function as antioxidants, and the increased levels of polyphenols and flavonoids in Kocuria-treated plants may protect the plant cellular components from oxidative damage. Abiotic stresses, such as drought, activate the phenylpropanoid pathway in plants and stimulate the accumulation of polyphenolic compounds. These compounds play a role in scavenging ROS, neutralizing free radicals, stabilizing cell membranes, and osmotic changes [34]. Kocuria may be involved in regulating the plant phenylpropanoid pathway via signaling molecules.
The PGP effects of Kocuria have been reported on crops other than wheat. For example, promotion of plant growth under salt stress has been described with Kocuria erythromyxa EY43 on strawberries [35], Kocuria rhizophila Y1 on maize [6], Kocuria arsenatis ST19 on tomato [7], and Kocuria kristinae on rice [36]. Kocuria erythromyxa Rt5M10 was found to promote the growth of grape vines with increased ROS-scavenging activity and accumulation of terpene compounds in the vine leaves [37]. The role of Kocuria in alleviating drought stress in wheat has remained largely unexplored. The dual stress tolerance (osmotic and UV) exhibited by Kocuria strains is especially valuable for field applications. Very often drought stress coincides with high solar radiation and inoculants must survive both the soil environment and the surface exposure period before colonizing roots. PGPB that can form stable association with roots are expected to exert beneficial effects over extended periods through multiple mechanisms such as production of IAA, nitrogen fixation, enhanced nutrient uptake etc. Both Kocuria strains showed a 2–2.8-fold greater abundance in the root-associated region of the plants. While our enumeration-based methods confirm increased bacterial numbers associated with roots, future studies using confocal laser scanning microscopy would provide valuable spatial information about colonization patterns, including endophytic versus epiphytic localization and preferential colonization zones.
KPC and KAD demonstrated the highest combined tolerance to osmotic stress (30%–40% PEG-6000), UV radiation (40 minutes exposure), and sustained PGP activity under drought conditions as compared to non-carotenoid-producing isolates (CMG-1, MAN, ANK-6, and FS-1). The basis for this is probably carotenoid-mediated protective functions. Several Kocuria species are known to synthesize carotenoids that protect bacterial cells from oxidative and environmental stress [38–42]. Carotenoids quench singlet oxygen through energy transfer and physically dissipate excess excitation energy, thereby preventing cellular damage [43]. This explains why KPC and KAD maintained high viability (7–8 × 10⁶ cfu/ml) after 15 minutes of UV exposure, while non-pigmented strains showed 10–100-fold reductions.
Carotenoids stabilize membranes under osmotic stress. The rigid isoprene structure of carotenoids integrates into lipid bilayers, reducing membrane fluidity and preventing water loss. This is vital for bacterial survival under drought conditions [44,45]. This membrane-stabilization by carotenoids may contribute to the PGP activities (IAA production, nutrient solubilization) observed in Kocuria strains even at 40% PEG-6000. The other strains that did not produce carotenoids did not exhibit plant growth promotion at 40% PEG-6000.
Drought stress induces oxidative stress in both bacteria and plants through disruption of electron transport chains and accumulation of ROS [46]. By scavenging ROS, carotenoids help preserve the function of many enzymes involved in metabolic pathways and thus enable continued IAA production and other PGP activities under stress conditions. The enhanced performance of Kocuria-treated plants may partly be attributed to carotenoid pigment production by K. rosea and K. turfanensis. Bacterial carotenoids can influence plant responses through multiple mechanisms. Apocarotenoids such as β-cyclocitral, β-ionone and dihydroactinidiolide are derived from carotenoids by oxidative cleavage [47].
Carotenoid-derived signalling molecule, β-cyclocitral regulates plant root architecture and growth [48]. Apocarotenoids, β-ionone and dihydroactinidiolide, enhance plant response to stresses other than drought. In addition, carotenoid-deficient bacterial mutants have been shown to exhibit reduced IAA production, impaired biofilm formation, and diminished root colonization ability [49]. These findings support the hypothesis that carotenoid production by Kocuria spp. contributes to their effective plant–microbe interactions and drought stress mitigation.
This study is the first report of Kocuria-mediated drought tolerance in wheat (T. durum). Since wheat is an important staple crop and is vulnerable to drought, this finding has significant agricultural implications, particularly for semi-arid regions of India. There is a need to further investigate the correlation between bacterial carotenoid production and combined tolerance to osmotic stress, UV radiation, and drought conditions. Carotenoid biosynthesis capacity could probably serve as a rapid screening criterion for identifying potential PGPB candidates suitable for field application in drought-prone environments.
Many PGPB show promise under laboratory conditions but do not perform well under field conditions. Using these two laboratory Kocuria cultures to develop bioinoculants for field application will require optimization of carrier materials, storage conditions, and application protocols. It may also be possible to employ these Kocuria strains in combination with other existing sustainable agricultural practices.
5. CONCLUSION
The present study demonstrates that the two pigment-producing isolates, K. turfanensis and K. rosea, effectively alleviate drought-induced stress in wheat. The combined tolerance to osmotic and UV stress, plant growth-promotion under stress, root association, and induction of plant protective responses, such as production of enhanced chlorophyll along with antioxidants and reduced ROS, make these strains valuable candidates for agricultural development. The application of Kocuria spp. as PGP bioinoculants, therefore, holds promise for improving wheat resilience and productivity, particularly in drought-prone regions.
6. ACKNOWLEDGMENTS
The authors gratefully acknowledge the Department of Microbiology and the Caius Research Laboratory, St. Xavier’s College, for providing access to essential instrumentation supported through the DST–FIST and DBT–BUILDER grants. This research was financially supported by the Seed Grant of St. Xavier’s College (Grant No. 001, 2024) and the Department of Biotechnology, Government of India, under the DBT–BUILDER program (Grant No.BT/INF/22/SP41293/2020). We thank Vishwas Sarangdhar for his valuable and constructive suggestions and useful critiques of this research work.
7. AUTHOR CONTRIBUTIONS
All authors made substantial contributions to conception and design, acquisition of data, or analysis and interpretation of data; took part in drafting the article or revising it critically for important intellectual content; agreed to submit to the current journal; gave final approval of the version to be published; and agreed to be accountable for all aspects of the work. All the authors are eligible to be authors as per the International Committee of Medical Journal Editors (ICMJE) requirements/guidelines.
8. CONFLICTS OF INTEREST
The authors declare that there are no conflicts of interest or competing financial or nonfinancial interests related to this study.
9. ETHICAL APPROVALS
This study does not involve experiments on animals or human subjects.
10. DATA AVAILABILITY
All the data are available with the authors and shall be provided upon request.
11. PUBLISHER’S NOTE
All claims expressed in this article are solely those of the authors and do not necessarily represent those of the publisher, the editors, or the reviewers. This journal remains neutral concerning jurisdictional claims in published institutional affiliation.
12. USE OF ARTIFICIAL INTELLIGENCE (AI)-ASSISTED TECHNOLOGY
The authors declare that they have not used AI tools for writing and editing of the manuscript, and no images were manipulated using AI.
REFERENCES
1. Chowdhury G, Saha AK Analysing agricultural distress in the eastern plateau of West Bengal's Rarh Region: integrating hybrid deep ensemble and GIS-based soft computing. Discov Appl Sci 2025;7:664; CrossRef
2. Ganguly A, Chattopadhyay S. Climate variability and drought assessment of Marathwada and Vidarbha Regions of Maharashtra. IJSTE 2021;8(5):1–7.
3. Fadiji AE, Santoyo G, Yadav AN, Babalola OO. Efforts towards overcoming drought stress in crops: revisiting the mechanisms employed by plant growth-promoting bacteria. Front Microbiol 2022;13:962427; CrossRef
4. Glick BR. Plant growth-promoting bacteria: mechanisms and applications. Scientifica 2012;963401; CrossRef
5. Fiodor A, Singh S, Pranaw K. The contrivance of plant growth promoting microbes to mitigate climate change impact in agriculture. Microorganisms 2021;9(9):1841; CrossRef
6. Li X, Sun P, Zhang Y, Jin C, Guan C. A novel PGPR strain Kocuria rhizophila Y1 enhances salt stress tolerance in maize by regulating phytohormone levels, nutrient acquisition, redox potential, ion homeostasis, photosynthetic capacity and stress-responsive genes expression. Environ Exp Botany 2020;174:104023; CrossRef
7. Dif G, Belaouni HA, Goudjal Y, Yekkour A, Djemouai N, Zitouni A. Potential for plant growth promotion of Kocuria arsenatis strain ST19 on tomato under salt stress conditions. South Afr J Bot 2021;138:94–104; CrossRef
8. Nautiyal CS. An efficient microbiological growth medium for screening phosphate solubilizing microorganisms. FEMS Microbiol Lett 1999;170(1):265–70; CrossRef
9. Kumar A, Singh S, Mukherjee A, Rastogi RP, Verma JP. Salt-tolerant plant growth-promoting Bacillus pumilus strain JPVS11 to enhance plant growth attributes of rice and improve soil health under salinity stress. Microbiol Res 2021;242:126616; CrossRef
10. Olagunju OO, Ogunnusi TA, Akpor OB. Evaluation of Indole acetic acid and hydrogen cyanide production. Vegetos 2026;39:582–589; CrossRef
11. Travnickova E, Mikula P, Oprsal J, Bohacova M, Kubac L, Kimmer D, et al. Resazurin assay for assessment of antimicrobial properties of electrospun nanofiber filtration membranes. AMB Express 2019;9(1); CrossRef
12. Niu X, Song L, Xiao Y, Ge W. Drought-tolerant plant growth-promoting rhizobacteria associated with foxtail millet in a semi-arid and their potential in alleviating drought stress. Front Microbiol 2018;8:2580; CrossRef
13. Munsch-Alatossava P, Rita H, Alatossava T. A faster and more economical alternative to the standard plate count (SPC) method for microbiological analyses of raw milks. I AMV, redaktör, Communicating current research and educational topics and trends in applied microbiology. Badajoz: Formatex 2007;495–9. (Microbiology series).
14. Kumari S, Vaishnav A, Jain S, Varma A, Choudhary DK. Induced drought tolerance through wild and mutant bacterial strain Pseudomonas simiae in mung bean (Vigna radiata L.). World J Microbiol Biotechnol 2016;32; CrossRef
15. Kasim WA, Osman MEH, Omar MN, Salama S. Enhancement of drought tolerance in Triticum aestivum L. seedlings using Azospirillum brasilense NO40 and Stenotrophomonas maltophilia B11. Bull Nat Res Centre 2021;45(1); CrossRef
16. Li J, Yu G, Wang X, Guo C, Wang Y, Wang X. Jasmonic acid plays an important role in mediating retrograde signaling under mitochondrial translational stress to balance plant growth and defense. Plant Communications 2025;6(1); CrossRef
17. Marjanovic A, Djedjibegovic J, Lugusic A. et al. Multivariate analysis of polyphenolic content and in vitro antioxidant capacity of wild and cultivated berries from Bosnia and Herzegovina. Sci Rep 2021;11:19259; CrossRef
18. Attard E. A rapid microtitre plate Folin-Ciocalteu method for the assessment of polyphenols. Cent Eur J Biol 2013;8:48–53; CrossRef
19. Yadav P, Malpathak N. Estimation of antioxidant activity and total phenol, flavonoid content among natural populations of caper (Capparis moonii, Wight) from Western Ghats region. Indian J Pharm Educ Res 2016;50(3):495–501; CrossRef
20. Lo S, Nalawade SM, Mulabagal V, Matthew S, Chen C, Kuo C, et al. In vitro propagation by asymbiotic seed germination and 1, 1-Diphenyl- 2-picrylhydrazyl ( DPPH) radical scavenging activity studies of tissue dendrobium. Biol Pharm Bull 2004;27(5):731–5.
21. Xiong H, Hua L, Reyna-Llorens I, Shi Y, Chen KM, Smirnoff N, et al. Photosynthesis-independent production of reactive oxygen species in the rice bundle sheath during high light is mediated by NADPH oxidase. Proc Nat Acad Sci United States Am 2021;118(25):1–10; CrossRef
22. Rakhmawatie MD, Wibawa T, Lisdiyanti P, Pratiwi WR, Mustofa. Evaluation of crystal violet decolorization assay and resazurin microplate assay for antimycobacterial screening. Heliyon 2019;5(8):2263; CrossRef
23. Agarwal R, Kalambe SC, Chakraborty P, Chowdhury SR, Pant HJ. Biofouling reduction of EPDM by radiation-assisted modification for water environment applications. Appl Polym Sci 2024;141(5):e54871; CrossRef
24. Bolyen E, Rideout JR, Dillon MR, Bokulich NA, Abnet CC, Al-Ghalith GA, et al. Reproducible, interactive, scalable and extensible microbiome data science using QIIME 2. Nat Biotechnol 2019;37(8):852–7; CrossRef
25. Callahan BJ, Mcmurdie PJ, Rosen MJ, Han AW, Johnson AJ, Holmes SP. DADA2: high-resolution sample inference from Illumina amplicon data. Nat Methods 2016;13(7):581–3; CrossRef
26. Koshti R, Jagtap A, Noronha D, Patkar S, Nazareth J, Paulose R, et al. Evaluation of antioxidant potential and UV protective properties of four bacterial pigments. Microbiol Biotechnol Lett 2022;50(3):375–86; CrossRef
27. Vargas-García MC, López MJ, Elorrieta MA, F Suárez F, Moreno J. Physiology of exopolysaccharide production by Azotobacter vinelandii from 4-hydroxybenzoic acid. J Ind Microbiol Biotechnol 2002;29:129–33; CrossRef
28. Bhagat N, Raghav M, Dubey S, Bedi N. Bacterial exopolysaccharides: insight into their role in plant abiotic stress tolerance. J Microbiol Biotechnol 2021;31(8):1045–59; CrossRef
29. Banerjee A, Supakar S, Banerjee R. Melanin from the nitrogen-fixing bacterium Azotobacter chroococcum: a spectroscopic characterization. PLoS One 2014;9(1):e84574; CrossRef
30. Muñoz-Torres P, Cárdenas-Ninasivincha S, Aguilar Y. Exploring the agricultural applications of microbial melanin. Microorganisms 2024;12(7); CrossRef
31. Etesami H, Glick BR. Bacterial indole-3-acetic acid: a key regulator for plant growth, plant-microbe interactions, and agricultural adaptive resilience. Microbiol Res 2024;281:127602; CrossRef
32. Sharma A, Das N, Pandey P, Shukla P. Plant-microbiome responses under drought stress and their metabolite-mediated interactions towards enhanced crop resilience. Curr Plant Biol 2025;43:100513; CrossRef
33. Fang Y, Xiong L. General mechanisms of drought response and their application in drought resistance improvement in plants. Cellular Mol Life Sci 2015;72(4):673–89; CrossRef
34. Rao MJ, Zheng B. The role of polyphenols in abiotic stress tolerance and their antioxidant properties to scavenge reactive oxygen species and free radicals. Antioxidants 2025;14(1); doi: https://doi.org/10.3390/antiox14010074
35. Karlidag H, Yildirim E, Turan M, Pehluvan M, Donmez F. Plant growth-promoting rhizobacteria mitigate deleterious effects of salt stress on strawberry plants (Fragaria × ananassa). HortScience 2013;48(5):563–7; CrossRef
36. Pati B, Padhi S. Indole-3Acetic acid production by plant growth promoting rhizobacteria of saline soil, Odisha and its role in root elongation in rice plant. Scholars Acad J Biosci 2022;10(5); CrossRef
37. Salomon MV, Purpora R, Bottini R, Piccoli P. Rhizosphere associated bacteria trigger accumulation of terpenes in leaves of Vitis vinifera L. cv. Malbec that protect cells against reactive oxygen species. Plant Physiol Biochem 2016;106:295–304; CrossRef
38. Jagannadham MV, Rao VJ, Shivaji S. The major carotenoid pigment of a psychotrophic Micrococcus roseus strain: purification, structure, and interaction with synthetic membranes. J Bacteriol 1991;173(24):7911–7; CrossRef
39. Reddy GSN, Prakash JSS, Prabahar V, Matsumoto GI, Stackebrandt E, Shivaji S. Kocuria polaris sp. nov., an orange-pigmented psychrophilic bacterium isolated from an antarctic cyanobacterial mat sample. Int J Systematic Evol Microbiol 2003;53(1):183–7; CrossRef
40. Mulik A, Kumbhar P, Bhadekar R. Production and partial characterization of pigments produced by Kocuria Sp Bri 36: influence of heavy metals. Int J Pharm Pharm Sci 2017;9(10):137; CrossRef
41. Mal SA, Ibrahim GS, Al Khalaf MI, Al-Hejin AM, Bataweel NM, Abu-Zaid M. Production and partial characterization of yellow pigment produced by Kocuria flava isolate and testing its antioxidant and antimicrobial activity. Int J Life Sci Pharma Res 2022;10(2):58–66; CrossRef
42. Metwally RA, El-Sersy NA, El Sikaily A, Sabry SA, Ghozlan HA. Optimization and multiple in vitro activity potentials of carotenoids from marine Kocuria sp. RAM1. Sci Rep 2020;10:330; CrossRef
43. Maoka T. Carotenoids as natural functional pigments. J Nat Med 2020;74(1):1–6; CrossRef
44. Seel W, Baust D, Sons D, Albers M, Etzbach L, Fuss J, et al. Carotenoids are used as regulators for membrane fluidity by Staphylococcus xylosus. Sci Rep 2020;10(1):330; CrossRef
45. Kumar SV, Taylor G, Hasim S, Collier CP, Farmer AT, Campagna SR, et al. Loss of carotenoids from membranes of Pantoea sp. YR343 results in altered lipid composition and changes in membrane biophysical properties. Biochim Biophys Acta Biomembr 2019;1861(7):1338–45; CrossRef
46. Miller G, Suzuki N, Ciftci-Yilmaz S, Mittler R. Reactive oxygen species homeostasis and signaling during drought and salinity stresses. Plant Cell Environ 2010;33(4):453-67.; CrossRef
47. Liang MH, He YJ, Liu DM, Jiang JG. Regulation of carotenoid degradation and production of apocarotenoids in natural and engineered organisms. Crit Rev Biotechnol 2021;41(4):513–34; doi: https://doi.org/10.1080/07388551.2021.1873242.
48. Carnà M, Korwin Krukowski P, Tosato E, D’Alessandro S. Apocarotenoids as stress signaling molecules in plants. Agriculture 2025;15(9):926; CrossRef
49. Bible AN, Fletcher SJ, Pelletier DA, Schadt CW, Jawdy SS, Weston DJ, et al. A carotenoid-deficient mutant in Pantoea sp. YR343, a bacteria isolated from the rhizosphere of Populus deltoides, is defective in root colonization. Front Microbiol 2016;7:1–5; CrossRef
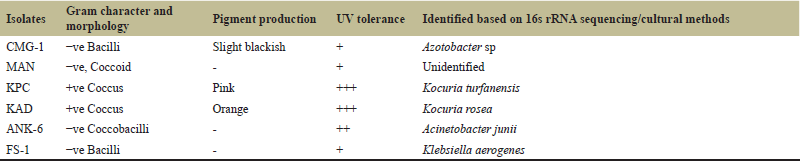 | Supplementary Table 1. Identification of isolates based on phenotypic traits and 16S rRNA gene sequencing. [Click here to view] |
| Supplementary Figure 1. Effect of bacterial inoculation on plant growth under controlled conditions (A) Growth of plants inoculated with bacterial isolates KPC, KAD, ANK-6, FS-1, and CMG-1. (B) Representative harvested plants from pots inoculated with KPC and KAD, compared with uninoculated plants from the well-watered control (CW) and uninoculated plants from the pots subjected to alternate-day watering (CWW). (C) Experimental setup showing plants grown under 80 W artificial light with a 12 hours light/12 hour dark photoperiod. [Click here to view] |