
1. INTRODUCTION
The concept of endophytes was introduced by De Bary [1] and refers to microorganisms that colonize the internal tissues of living plants without causing visible disease symptoms. Since the term “symbiosis” was introduced, numerous forms of symbiotic interactions have been identified among living organisms. The term is described as “the mutual living of dissimilar organisms” [2]. These definitions have been established based on fitness benefits or impacts on both microscopic symbionts and macroscopic hosts [3]. The mutualistic relationship fungi possess with plant species has grown to be one of the major concerns in biology. Fungal species classified as endophytic reside in plant tissues throughout their life cycle or a specific portion of it without producing visible signs of disease. These fungi mostly inhabit the inter or intracellular spaces of the host plants in many organs, including the leaf, root, stem, fruit, flower, and seed. Most investigated plant species, harbor endophytes, yet only a small fraction of the endophytic fungi associated with the world’s plant diversity has been characterized, suggesting that plants represent an immense and largely untapped reservoir of microbial diversity and biotechnological potential. Endophytic fungi have gained increasing attention since they have huge potential to produce a wide variety of metabolites that are significant for medicine [4].
Only a small number of these phytobiome-associated fungal endophytes have been investigated, suggesting that there is a good chance of discovering fascinating endophytes among a wide variety of plants in various niches and habitats. In addition, research on plant endophytes is required to furnish basic data for evaluating fungal diversity and distribution worldwide and for the identification of new species. Endophytic fungi inhabit plant tissues and establish symbiotic associations with their hosts, contributing to plant growth and development, enhancing tolerance to biotic and abiotic stresses, and stimulating the production of secondary metabolites [5,6]. Host plants along with their microbiota are referred to as holobionts. Certain endophytes may have developed as holobionts alongside their host and may have important implications for agriculture, medicine, or the environment [7–8]. Numerous studies have demonstrated that nearly all plants are colonized by endophytic fungi. Fungal diversity in plants has been influenced by a variety of parameters, such as host plant species, organs, geographic location, seasonal environment, and more [9].
Ascomycota, Basidiomycota, Mucoromycota, Glomeromycota, and Chytridiomycota are the current fungal taxa that have been documented to be endophytes of various plant species [10]. Numerous endophytic fungal species and a wide variety of metabolites with various purposes have been found in recent investigations [11–13]. They may also function as biocontrol agents [14], promote plant growth and generate enzymes [15]. Due to their relative underuse, endophytic fungi may provide a wide range of novel products that could be used in industry, the agricultural sector, as well as in medicines [16]. Abiotic and biotic stresses such as drought, heavy metals, salt, and other environmental pollutants such as floods, extremely high or low temperatures, predators, and infections can be mitigated by these endophytes. In addition to offering stimulants for plant growth and development, they confer advantageous biological characteristics on their hosts, including the ability to ward off harmful bacteria, insects, and other herbivores [17].
Endophytes have gained much attention as they produce valuable compounds. In order to find natural molecules that can be used as agrochemicals, researchers have been investigating secondary metabolites produced from these endophytes. Various chemicals have been extracted and isolated using top–down techniques from certain taxonomic orders of fungi [18]. A study reported that remarkable diversity of bioactive compounds, including glucosides, cytochalasans, azaphilones, terpenoids, nonribosomal peptides, macrolide polyketides, benzenoids, and lactones from Xylariales [18]. Endophytic fungi are relatively unknown sources of innovative natural compounds with uses in industry and agriculture. In fact, a variety of chemicals produced by endophytes have therapeutic utility [19]. The present review gives readers an overview of endophytic fungi, discovers the remarkable diversity of endophytic fungi, their distribution, function, and immense biological potential. Thus, the variety and biogeography of endophytic fungal communities, as well as their potential to support the sustainability of the agro-environment, are the primary subjects of this article. It also suggests potential paths to close the knowledge gaps and encourages more investigations.
2. DIVERSITY, TAXONOMY, AND BIOGEOGRAPHY OF ENDOPHYTIC FUNGAL COMMUNITIES
The variety of fungal endophytes within the tissues of plants can differ even among species, depending on the physiological conditions of each individual plant [20]. As a result, the variety of plant-associated fungal endophytes varies considerably [9]. Furthermore, the population profile of these fungi might be influenced by the age of the plant. Certain fungal endophytes can colonize a wide variety of plant species, while others are highly specialized and can only be found inside a small number of plants. This specialization may also exist with respect to the area of the plant that has been colonized [21]. In contrast to horizontally transmitted fungi, which are more probably to be antagonists, vertically transmitted fungi appear to exhibit plant interactions with a more mutualistic profile [9]. To maintain ecosystem functioning and variety across a wide range of plant species, it is imperative to do research on the endophytic fungal community in an evolutionary framework [22].
Research on the distribution and variety of endophytic fungi has been conducted throughout a broad range of geographical areas, including freshwater, marine, terrestrial, and semi-aquatic settings. Likewise, a wide range of phototrophs, including forest trees, mangroves, ferns, medicinal plants, seaweeds, vegetables, seagrass, and orchids, have been checked for endophytic fungi. The variety of these endophytes also varies substantially based on the location and is influenced by a variety of factors, including the growth season, anthropogenic effects, host plant physiology and genotype, and the environment. It varies greatly in abundance and variety among host plants, even within the same geographic region, and even inside the same host plant [23–24]. It was observed that, in comparison to other places, the fungal diversity is significantly higher in tropical and subtropical areas [25–26]. Seasonal fluctuations have also been identified as a significant factor influencing the variety and spread of these endophytes. The focus of endophytic fungal research has primarily shifted from taxonomic novelty to applications. It has been noted that numerous fungal endophytes are unknown to science [27]. Even though fungal endophytes are abundant and diverse throughout a wide range of biomes, research on their uses and functions is still in its early stages.
2.1. Taxonomic Basis of Endophytic Fungi
Fungal endophytes are commonly classified according to their phylogeny, host range, tissue colonization pattern, and mode of transmission [12–28]. Based on phylogenetic relationships, they are broadly categorized into clavicipitaceous (Class 1) and non-clavicipitaceous (Classes 2–4) endophytes. Clavicipitaceous endophytes are predominantly associated with cool-season grasses and exhibit a relatively narrow host range, whereas non-clavicipitaceous endophytes colonize a broad spectrum of vascular plants and inhabit various internal tissues, including leaves, stems, roots, and seeds [28]. Endophytic fungi may also be classified according to the plant organ they colonize, such as foliar, root, stem, or seed endophytes, and by their mode of transmission as vertically transmitted (seed-borne) or horizontally transmitted (environmentally acquired) [12–27]. By definition, endophytic fungi inhabit living plant tissues without causing visible disease symptoms for at least a part of their life cycle, although certain species may transition to latent pathogenic, saprotrophic, or mutualistic lifestyles in response to host developmental stage or environmental conditions [28–29]. Unlike saprotrophs, which derive nutrients from dead organic matter, necrotrophic fungi are pathogens that actively kill host cells and subsequently utilize the dead tissues as a nutrient source; therefore, necrotrophy should not be considered a nutritional strategy of endophytic fungi [5–30].
2.2. Distribution of Fungal Endophytes in the Terrestrial Habitat
Being a varied and diverse guild in ecology, an endophytic fungus possesses a huge range of functional features related to host phytogeography, adaptation, and defense. Fungal endophytes have been distributed in the terrestrial habitat and share niches with trees, orchids, shrubs, medicinal plants, ferns, etc. (Fig. 1). Arnold and Lutzoni [31] recognized tropical trees and their leaves as unique hotspots with a wide diversity of endophytes based on the amount of mutualistic fungal colonization. The endophytic fungal diversity in the dry tropics was not particularly great, regardless of the type of habitat or tree species; nonetheless, there is a tendency toward the dominance of a small number of core group fungi, such as Colletotrichum, Pestalotiopsis, Phomopsis, and Xylaria [32]. In two dry tropical forests in southern India, 24 tree hosts from 17 families revealed 81 endophytes in 3,600 segments [33]. In northern China, 2,065 endophytes isolated from 4,320 tissue sections of Pinus tabulaeformis [34]. Twenty-six fungal endophytes were reported from Juniperus procera in Saudi Arabia [35].
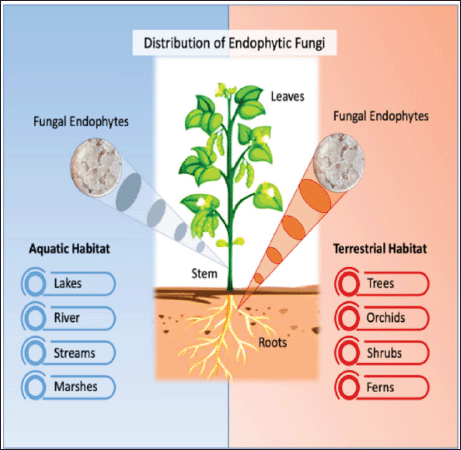 | Figure 1. Distribution of endophytic fungi. [Click here to view] |
There are numerous cases where the fungi live in association with plants of medicinal importance and create some of the value-added compounds [36–37]. Based on morphological and genetic approaches, 46 endophytic fungi were found in the foliar section of six medicinal herbs from central India, whereas 34 fungal species were found in three medicinal shrubs [38]. Eleven species of aquatic hyphomycetes as endophytes have been identified by Sati and Belwal [39] in the roots of numerous riparian pteridophytes at two places in Kumaun, Himalaya. There is little information available about endophytic fungi, despite the fact that orchids must be in close proximity to fungi in order to meet their nutritional and seed germination needs [40–41]. To learn more about orchids’ relationship with mycorrhizal fungi, evaluations of up to 200 genera of orchids have been conducted [42]. Thirty-three samples of roots and tubers from five different species of Mediterranean orchids were examined, and Fusarium, Papulaspora, and Rhizoctonia were identified [43]. The orchid Odontoglossum sp. was shown to harbor endophytic Phomopsis sp. in Northern Ecuador [44]. Anoectochilus setaceus, a type of orchid found in Sri Lanka, included the endophytic Xylaria sp. [45]. Endophytic fungi were evaluated in 90 segments of two major orchid species from the Western Ghats of India, Bulbophyllum neilgherrense and Vanda testacea [46]. Further, considerable numbers of fungi were recorded in the leaf segments of both orchids rather than in the bulb, stem, or roots.
2.3. Distribution of Fungal Endophytes in the Aquatic Habitat
Research on the distribution and diversity of endophytic fungi in aquatic habitats is rather rare [47]. Compared to terrestrial and marine areas, less research has been done on endophytic fungi in freshwater environments. A variety of plant species are influenced by freshwater environments, including lakes, rivers, streams, and marshes (Fig. 1). Numerous species of riparian trees extend their roots into flowing waters that could be possible sites for fungal colonization. This hinders the complete elimination of fungi from higher portions of streams and rivers. The endophytic stage of two common aquatic hyphomycetes (Campylospora parvula and Tricladium splendens) was initially shown by Fisher and Petrini in 1989. The occurrence of Filosporella fistucella, Fontanospora fusiramosa, Filosporella versimorpha and Tetracladium nainitalense as endophytes of riparian plants has subsequently been documented by Sati and Belwal [39]. In tropical and subtropical climates, plant varieties found in river mouths (estuaries and mangroves) offer possible sites for endophytic fungi colonization. In mangrove plant species found along India’s east coast, common foliar endophytes are Acremonium, Phomopsis, Phyllosticta, and Sporormiella minima. There are 619 endophytic fungi on Thai mangrove trees, with Bruguiera cylindrica having the highest colonization [48]. Twenty-five endophytic fungi were isolated from the mangrove shrub and fern, which include Acanthus ilicifolius and Acrostichum aureum, respectively [49].
Sesbania bispinosa, a mangrove legume native to southwest India, contained 25 endophytic fungi, the majority of which were found in the root segments [50]. A study reported that fungal species of the wild legume S. bispinosa, which is acclimated to mangroves and coastal sand dunes [51]. Worldwide, seaweeds are home to about 100 known endophytic fungi, of which up to 75% have been documented from the North Sea, the Baltic Sea, Canada, the United Kingdom, India, and China [52]. The diversity of fungal endophytes associated with red, brown, and green seaweeds from the coastal areas of India has been comprehensively compiled and discussed [53]. The east coast of India Halophila ovalis revealed a low colonization density of 14 endophytic fungi in its petiole, rhizome, and leaf blade [54]. The endophytic fungi inhabiting the leaf tissues and rhizomes of ten seagrass species collected from the east coast of India were examined by Venkatachalam et al. [55]. Three seagrass species, Zostera japonica, Zostera marina, and Thalassia testudinum gathered from Hong Kong (China), and the Philippines, are reported to have approximately 26 endophytic fungi [56].
3. SPECIFIC BIOACTIVE METABOLITES PRODUCED BY ENDOPHYTIC FUNGI
The ability of endophytic fungi to produce secondary metabolites that are precious for the manufacturing of novel drugs makes them of biotechnological interest [57]. It is thought that these fungi are a good source of novel bioactive substances [58]. They have been found to produce bioactive compounds, including resveratrol, taxol, podophyllotoxin, huperzine, and vinca alkaloids [59–60]. These compounds have the potential to be used as therapeutic agents for the treatment of a variety of illnesses, either directly or indirectly [61]. Steroids, alkaloids, phenols, isocoumarins, xanthones, quinones, and terpenoids are some secondary metabolites produced by endophytic fungi [62–63] (Table 1). Novel, advantageous bioactive compounds with biological properties [64] such as antituberculosis [65], antiinflammatory [66], antiprotozoal [67], insecticidal [68], antiviral, anticancer activities [69], immunomodulatory [70], and anthelmintic activity [62] have been reported in a number of studies. Abundant pharmacologically significant compounds, including the antimicrobial metabolite 5α,8α-epidioxyergosta-6,22-dien-3β-ol [71], the anticancer cajanol [72], the podophyllotoxin and kaempferol [73], the antiinflammatory ergoflavin [74], the antioxidant lectin [75], the insecticidal heptelidic acid [76], the immunosuppressive sydoxanthone A, B [77], and the cytotoxic radicicol [78] were produced by fungal endophytes. Various enzymes with important clinical and industrial applications, including lipases, amylases, catalases, laccases, and proteases, have also been reported from endophytic fungi.
4. ROLE OF FUNGAL ENDOPHYTES IN BIOLOGICAL ACTIVITIES
It has been discovered that endophytic fungi are a novel source of bioactive secondary metabolites with a wide range of biological activities, including biocontrol activities, antibiotic production, immunosuppressive, antimycotic, and anticancerous activities. They play an important role as plant growth promoters (PGP) [79] and help in nutrient recycling bioremediation and biotransformation (Fig. 2).
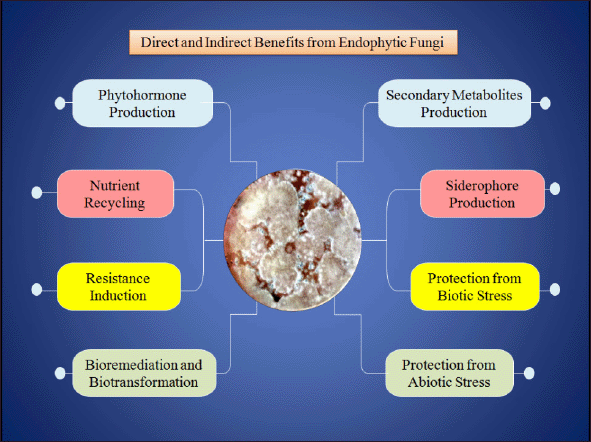 | Figure 2. Benefits provided by endophytic fungi. [Click here to view] |
4.1. Biological Control Agents
Biological control is the process of reducing the detrimental effects of plant pathogens and encouraging beneficial responses by the plant by utilizing beneficial organisms, their genes, and/or products, such as metabolites. Various crop plant varieties that were derived from wild types are used in current agricultural techniques. Since these crop plants cannot acquire resistance against the new pathogens, new pathogens may arise and occasionally trigger disease epidemics [80]. Excessive pesticide use lowers agricultural sustainability and has negative consequences for human health and ecological function. Agrochemicals deplete soil fertility, disrupt natural equilibrium, and pollute the environment and food chains [81].
Fungal entomopathogens are thought to be a diverse group of organisms on this planet, Earth, and are natural enemies of arthropods. They are the subject of extensive global research and have great potential as biocontrol agents. Adoption and application of these fungal entomopathogens in biocontrol is an alternative to chemical pesticides that harm the ecosystem [82]. The use of fungal biopesticides provides an environmentally friendly and highly efficient substitute. Endophytes have the capacity to modify their interactions with pathogens and pests and may even serve as potential biocontrol agents. Endophytic fungi can shield their host plant against insect infection by producing peramine, which prevents insects, nematodes, and other phytoparasites from eating the plant [83]. Important biocontrol agents include Aspergillus spp., Gliocladium spp., nonpathogenic Fusarium spp., Trichoderma spp. etc. Acremonium alternatum, an endophyte, protects Chinese cabbage from Plasmodiophora brassica [84].
A fungal endophyte called Phomopsis sp. was identified from cotton plants, and it helped the plants resist caterpillar herbivory [85]. Occasionally, a certain endophytic species shows promise as a biocontrol agent. Considering the added benefits; the same endophyte species may promote the growth of the host plant, fitness, and stress tolerance, and protect the host plant from pests and diseases. Endophytic fungi such as Aspergillus, Cladosporium, Paecilomyces, and Diaporthe were also found to be promising biocontrol agents against Duponchelia fovealis [86]. Endophytic fungal isolates obtained from T. wilfordii exhibited larvicidal activity against mosquito larvae. [87]. Cladosporium uredinicola has been reported to manage the population of Spodoptera litura. Sarocladium strictum also exhibits insecticidal properties against Spodoptera littoralis [88]. Acremonium vitellinum serves as a potential biocontrol agent against Helicoverpa armigera [89].
Species of Trichoderma can colonize a variety of crops, including cotton, soybeans, wheat, and corn. Although it demonstrates an impressive capacity to parasitize a wide range of plant infections, this fungus is most recognized for its ability to develop resistance in plants [90]. Furthermore, a number of strains have been documented to parasitize eggs and juveniles (second stage) of Meloidogyne javanica and the incredibly tough cysts of Heterodera avenae [91]. As a result, a variety of hosts are present for Trichoderma species, including plants and other plant pathogens that are parasitic or symbiotic, respectively. Purpureocillium lilacinum is a well-known biocontrol agent for insects and nematodes that parasitize plants. It has been reported as a promising nematicide to manage plant pathogenic nematodes [92]. It has also been found to manage the Blatta orientalis and Shelfordella populations under laboratory condition [93].
4.2. Antimicrobial Actions
Endophytic fungi have been discovered as a potent source of naturally occurring biomolecules that possess antimicrobial activities such as antioxidant, antibiotic, cytotoxic, antimalarial, antitumor, enzyme-inhibition, and anti-filarial activities [63]. These biomolecules are actually the secondary metabolites produced by endophytic fungi (Table 1). A number of metabolites isolated from fungal endophytes have shown antimicrobial properties. The leaf tissues of the medicinal plant Callistemon subulatus were used to isolate Aspergillus sp. ASCLA, which produces isoshamixanthone, and it showed antibacterial properties against pathogenic microorganisms [94]. Three novel α-pyrone derivatives were discovered from Penicillium ochrochloronthe, and these compounds have antibacterial action against some strains of pathogenic bacteria and fungi [95]. Ramos et al. [96] reported two endophytic fungi, namely Papulaspora immersa and Apiospora montagnei, from Smallanthus sonchifolius in Brazil; these endophytes showed antibacterial efficacy against a variety of test species in different extract forms. Aspergillus fumigatus was isolated from the leaves of Albizia lucidior [97] and Ocimum basilicum [98], and it may have antibacterial and antifungal properties against the majority of common resistant microorganisms. Colletotrichum gloeosporioides was also reported to have antibacterial activities against Bacillus subtilis, Staphylococcus aureus, Pseudomonas aeruginosa, and Escherichia coli and antimycotic activities against Candida albicans [99].
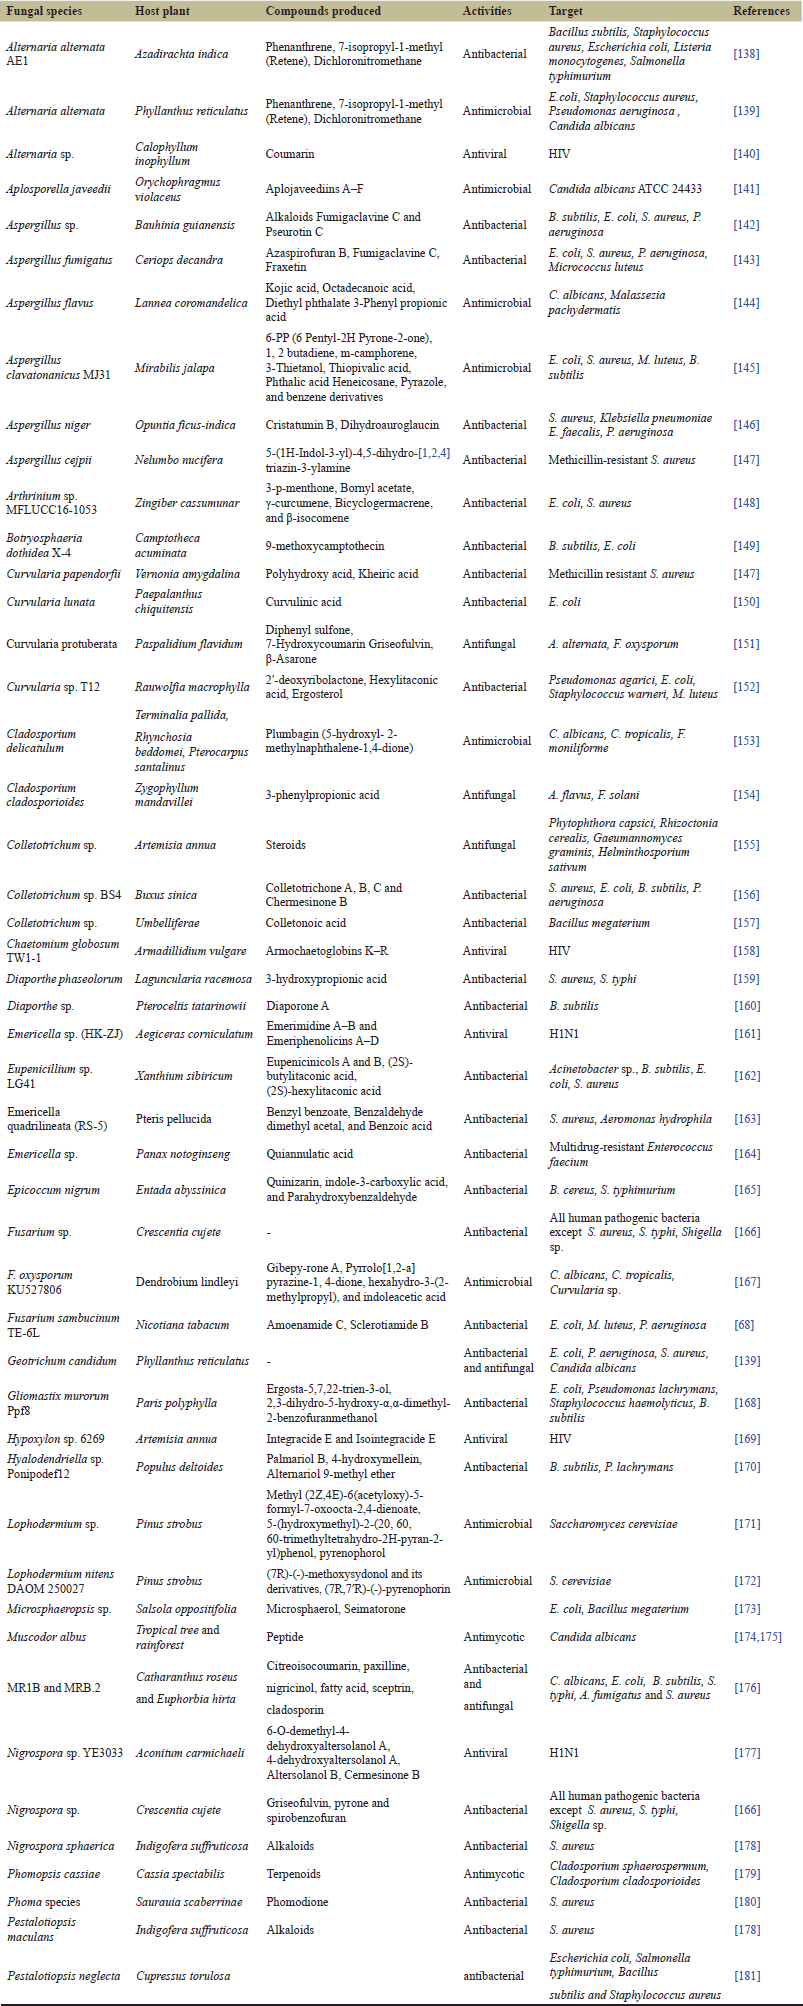 | Table 1. Secondary metabolites produced by endophytic fungi and their activities. [Click here to view] |
Alternaria alternata extract was obtained from Picrorhiza kurroa, possesses antioxidant and antibacterial action against S. aureus and B. subtilis [100]. Antibacterial and antifungal properties against B. subtilis, Bacillus cereus, C. albicans, S. aureus, S. typhimurium, E. coli, P. aeruginosa, and K. pneumoniae, were discovered in Aspergillus flavus [98]. Aspergillus nidulans, discovered in O. basilicum, also showed antimicrobial activities against several microorganisms [98]. Aspergillus welwitschiae, isolated from Aloe ferox, has potential antibacterial activity against disease-causing microorganisms [101]. Similarly, Penicillium citrinum isolated from Azadirachta indica also exhibits antimicrobial potential against human disease-causing bacteria and fungi [102]. The endophytic Aspergillus tubingensis has demonstrated potential antibacterial efficacy against gram-positive, gram-negative, and unicellular fungi. It may also prevent the production of biofilms [103]. Promising antimicrobial activities were observed from the endophytic Aspergillus niger against S. aureus, E. coli, P. aeruginosa, Micrococcus lutus, and C. albicans [104].
Stephania dielsiana exhibits the fungal endophyte Penicillium sp. that showed significant antimicrobial properties toward pathogenic bacteria [105]. The antimicrobial potential was also reported in the extracts of Penicillium funiculosum and Penicillium pinophilum [106,107]. Pathogenic microorganisms are susceptible to the antibacterial activity of Nigrospora spp. [108]. Emericella nidulans, which possesses potent antifungal activity against A. niger, Microsporum audouinii, and Penicillium sp. [109]. Antibacterial activities against B. cereus and Staphylococcus epidermidis were reported from Diaporthe sp. [110]. It was recently reported that nigranoic acid was extracted from an endophytic Trichoderma sp. and exhibited potent antiviral activity [111]. Pulchranin, an anticancer drug, was produced by the Aspergillus TRL1, was isolated from Tabebuia rosea. It was reported that this molecule effectively suppresses human tumor cells, including liver (Hep-G2) cell lines and breast (MCF-7) cell lines [112].
4.3. Production of Phytohormone and PGP
The interactions between the fungal endophytes and the host plants showed a neutral antagonism because the identification of the plant as a host necessitates the enactment of virulence factors for fungal colonization and the induction of host defenses by these processes [113]. This connection maintains equilibrium between fungi and host, since the fungus benefits the host plant by surviving on its resources and by providing resistance to both biotic and abiotic stresses [21]. The plant provides endophytes with a protected habitat, limited competition with other microbes, and the nutrients needed for fungal survival and growth [114]. Thus, through a variety of processes, fungi enhance plant fitness in return for this secure environment.
Recently, the use of endophytic fungi to stimulate plant growth has garnered attention due to the significant role these fungi play in increasing plant tolerance to both biotic and abiotic stressors and raising yield [115]. Through two primary pathways, that is, direct and indirect, these endophytes have considerable potential to cause PGP. Direct mechanisms include the synthesis of phytohormones and the uptake of nutrients. The production of antibiotics, siderophores, secondary metabolites, induced resistance, and defense against ecological stressors are included in the indirect mechanism [116]. Fungal endophytes can produce cytokinins, auxins, and gibberellins. Even though gibberellins are equally crucial to plant growth in many environmental situations as chemical signaling and messengers, the ability of endophytic fungi to produce phytohormones is understudied [117]. The primary auxin that fungi make is called indole-3-acetic acid (IAA). It is the primary controller of plant growth and is responsible for the growth of shoots and roots, including the commencement of the root formation process, vascular tissue differentiation, and tropism responses [118]. Gibberellins are necessary for a number of plant responses, including fruit production, senescence, flowering, stem elongation, sexual expression, and seed germination [119].
Purpureocillium lavendulum, P. lilacinum, and Metarhizium marquandii have been shown to produce IAA and solubilize phosphorus (P) from fluorapatite. After testing on plants of maize, beans, and soybeans, the colonization of these fungal endophytes was found to improve and enhance growth factors such as shoots and roots and nutrient availability such as sulfur (S) and nitrogen (N) [120]. In addition to increasing nitrogen fixation and phosphate solubilization, promoting the synthesis of siderophores, inhibiting ethylene production through the action of 1-aminocyclopropane-1-carboxylate (ACC) deaminase, and influencing enzyme synthesis, fungal endophytes can also have an impact on plant development by producing phytohormones [121–124].
Fungal endophytes such as those reported from Teucrium polium showed unpredictable ability for phosphate solubilization, which acts as a promising PGP [125]. Three fungal endophytes from Oryza coarctata, namely Talaromyces adpressus, Talaromyces argentinensis, and A. welwitschiae, have been reported in Bangladesh that exhibit PGP capability. IAA, ACC deaminase, and siderophore production were recorded from T. adpressus and T. argentinensis, along with phosphate, and zinc solubilization as well as N fixation under in vitro conditions having high salinity. Furthermore, A. welwitschiae showed improved metabolite and chlorophyll content [126]. Trichoderma longibrachiatum T6 has been documented to boost the plants’ tolerance to NaCl stress and encourage the growth of Triticum aestivum [124].
Macrophomina phaseolina isolate MP-1, Macrophomina phaseolina isolate MP-3, Diaporthe phaseolorum, Daldinia eschscholtzii, Trichoderma koningii, and Trichoderma erinaceum exhibited high phosphate-solubilizing ability and extracellular enzyme production under greenhouse conditions [127]. A study recorded that the biomass yield, nutritional value, and mineral status of Trifolium subterraneum feed were impacted by fungal endophytes; however, the impacts differed depending on the type of fungus. In the field, Chaetosphaeronema sp. boosted fodder productivity by about 80%. In the greenhouse experiment, Fusarium lateritium and Pleosporales decreased the concentration of aluminum, while Epicoccum nigrum decreased the lead content of the feed. Stemphylium globuliferum was the primary source of a rise in vital nutrients, such as zinc [128]. The application of Xylariaceae sp., Fusarium avenaceum, and Sarocladium terricola has been reported to enhance the germination of Lolium multiflorum seeds by over 70%. The use of fungus filtrates had a favorable effect on shoot and root length, plant dry weight, and root count [129].
Trichoderma species, Aspergillus flavus, Penicillium digitatum, Podospora bulbillosa, Actinomucor elegans, Gliocladium virens, Arbuscular mycorrhizal fungi, etc. have demonstrated their environmentally friendly ability to enhance crop production by promoting the growth of crop plants’ shoots and roots, seed germination, chlorophyll production for photosynthesis, and an abundance of crop yields [130]. Numerous studies have documented the benefits of fungal endophytes such as Gliocladium, Penicillium, Phoma, Phytophthora, Rhizoctonia, Talaromyces, Trichoderma in plant growth promotion. These genera have been shown to enhance the growth of orange, tomato, apple, pear, cucumber, carrot, and other plants, as well as to further support the innate immunity and the production of various necessary secondary metabolites by the plants [131–136]. Plant growth-promoting fungi (PGPF) enhance plant growth through phytohormone production, nutrient acquisition, induced systemic resistance, and suppression of phytopathogens [137].
5. FUTURE PROSPECT AND CHALLENGES
Endophyte-plant interactions can be used as an effective and reasonable integrated disease management technique and can be essential in promoting low-cost sustainable agriculture applications due to their substantial significance as a possible biocontrol agent. More knowledge of the metabolite structures created by endophytic fungi and plant support protection mechanisms may help with integrated management strategies. However, because of regulatory requirements, challenges with mass production, inoculant efficacy, and farmer and consumer resistance, their agricultural application is still restricted. The use of fungal endophytes can be employed by small marginal farmers, but it cannot be utilized for large-scale production. Particularly, in extreme habitats, the conflict between inoculated fungal endophytes and native microbiomes could result in adverse effects or lower efficacy. Several endophytes have been reported to enhance plant growth and productivity, but they also affect invertebrates and vertebrate species.
Researchers might be able to investigate and make extensive use of endophyte resources in the future. One option is to look for unique endophytes in plants that thrive under harsh conditions. Another is to look for appropriate and productive ways to extract more potent bioactive substances from a variety of endophytes. Ultimately, it will be promising for large-scale manufacturing to increase the yield and content of active compounds in recognized strains based on metabolic regulation and genetic engineering. Endophytes have only recently been investigated, despite the fact that fungi have been shown to be economically significant suppliers of enzymes for restoration of the environment and other applications. Endophytes are therefore a fascinating niche that is just waiting to be exploited.
6. CONCLUSION
Climate change, population expansion, and other stressors are posing growing concerns about global food security, highlighting the urgent need to increase agricultural yields in vulnerable areas. The study of fungal endophytes provides insight on the diversity, biogeography, and various biological activities of fungal endophytes. Endophytic fungi perform remarkable functions in the ecosystem, including abiotic and biotic stress tolerance, eco-adaptation, boosting growth and development, and maintaining the health of their host. It is an affordable and environmentally responsible alternative to increase food production and advance sustainable agricultural methods. Because they produce biologically active chemicals against both biotic and abiotic stresses by activating useful products for agricultural output under rapid climate change scenarios, fungal endophytes can be regarded as a crucial tool in regulating both types of stresses. Endophytic fungi are a valuable tool for research and businesses, as evidenced by their usage as an alternative with significant potential in the sectors of biocontrol, bioremediation, biotransformation, and biofertilization.
7. ACKNOWLEDGMENTS
The author acknowledges Eternal University, Baru Sahib, for providing necessary facilities to complete this work.
8. AUTHOR CONTRIBUTIONS
All authors made substantial contributions to conception and design, acquisition of data, or analysis and interpretation of data; took part in drafting the article or revising it critically for important intellectual content; agreed to submit to the current journal; gave final approval of the version to be published; and agree to be accountable for all aspects of the work. All the authors are eligible to be authors as per the International Committee of Medical Journal Editors (ICMJE) requirements/guidelines.
9. CONFLICTS OF INTEREST
The authors report no financial or any other conflicts of interest in this work.
10. FUNDING
There is no funding to report.
11. DATA AVAILABILITY
There are no available data or extra materials for this review.
12. PUBLISHER’S NOTE
All claims expressed in this article are solely those of the authors and do not necessarily represent those of the publisher, the editors and the reviewers. This journal remains neutral with regard to jurisdictional claims in published institutional affiliation.
13. USE OF ARTIFICIAL INTELLIGENCE (AI)-ASSISTED TECHNOLOGY
The authors declare that they have not used artificial intelligence (AI)- tools for writing and editing of the manuscript, and no images were manipulated using AI.
REFERENCES
1. de Bary A. Morphologie und Physiologie der Pilze, Flechten und Myxomyceten. Hofmeister’s handbook of physiological botany, Volume II. Engelmann, Leipzig, Germany, 1866. CrossRef
2. de Bary A. Die Erschenung Symbiose. In: Trubner KJ (ed.). Vortrag auf der Versammlung der Naturforscher und Artze zu Cassel, Verlag, Strasbourg, France, pp 1–3, 1879. CrossRef
3. Lewis DH. Symbiosis and mutualism: crisp concepts and soggy semantics. In: Boucher DH (ed.). Biology of mutualism, Croom Helm Ltd, London, UK, pp 29–43, 1985.
4. Kusari S, Zühlke S, Spiteller M. An endophytic fungus from Camptotheca acuminata that produces camptothecin and analogues. J Natural Prod 2009;72:2–7. CrossRef
5. Gupta S, Chaturvedi P, Kulkarni MG, Van Staden J. A critical review on exploiting the pharmaceutical potential of plant endophytic fungi. Biotechnol Adv 2020;39:107462. CrossRef
6. Hartley SE, Eschen R, Horwood JM, Gange AC, Hill EM. Infection by a foliar endophyte elicits novel arabidopside-based plant defence reactions in its host, Cirsium arvense. New Phytol 2015;205:816–27. CrossRef
7. Gouda S, Das G, Sen SK, Shin HS, Patra JK. Endophytes: a treasure house of bioactive compounds of medicinal importance. Front Microbiol 2016;7:1538. CrossRef
8. Vandana UK, Rajkumari J, Singha LP, Satish L, Alavilli H, Sudheer PD, et al. The endophytic microbiome as a hotspot of synergistic interactions, with prospects of plant growth promotion. Biology 2021;10:101. CrossRef
9. Aly AH, Debbab A, Proksch P. Fungal endophytes: unique plant inhabitants with great promises. Appl Microbiol Biotechnol 2011;90:1829–45. CrossRef
10. Abeywickrama P, Qian N, Jayawardena R, Li Y, Zhang W, Guo K, et al. Endophytic fungi in green manure crops; friends or foe. Mycosphere 2023;14(1):1–106. CrossRef
11. Xiao J, Zhang Q, Gao YQ, Tang JJ, Zhang AL, Gao JM. Secondary metabolites from the endophytic Botryosphaeria dothidea of Melia azedarach and their antifungal, antibacterial, antioxidant, and cytotoxic activities. J Agric Food Chem 2014;62:3584–90. CrossRef
12. Zimmerman NB, Vitousek PM. Fungal endophyte communities reflect environmental structuring across a Hawaiian landscape. Proc Nat Acad Sci 2012;109:13022–7. CrossRef
13. Zhang D, Ge H, Zou JH, Tao X, Chen R, Dai J. Periconianone A, a new 6/6/6 carbocyclic sesquiterpenoid from endophytic fungus Periconia sp. with neural anti-inflammatory activity. Org Lett 2014;16:1410–3. CrossRef
14. Adeleke BS, Ayilara MS, Akinola SA, Babalola OO. Biocontrol mechanisms of endophytic fungi. Egyptian J Biol Pest Control 2022 24;32(1):46. CrossRef
15. Baron NC, Rigobelo EC. Endophytic fungi: a tool for plant growth promotion and sustainable agriculture. Mycology 2022;2;13(1):39-55. CrossRef
16. Strobel G, Daisy B, Castillo U, Harper J. Natural products from endophytic microorganisms. J Nat Prod 2004;67:257–68. CrossRef
17. Sudha V, Govindaraj R, Baskar K, Al-Dhabi NA, Duraipandiyan V. Biological properties of endophytic fungi. Braz Arch Biol Technol 2016;59:16150436; e16150436. CrossRef
18. Becker K, Stadler M. Recent progress in biodiversity research on the Xylariales and their secondary metabolism. J Antibiot 2021;74:1–23. CrossRef
19. Kharwar RN, Mishra A, Gond SK, Stierle A, Stierle D. Anticancer compounds derived from fungal endophytes: their importance and future challenges. Nat Prod Rep 2011;28:1208–28. CrossRef
20. Vega FE, Simpkins A, Aime MC, Posada F, Peterson SW, Rehner SA, et al. Fungal endophyte diversity in coffee plants from Colombia, Hawai’i, Mexico and Puerto Rico. Fungal Ecol 2010;3:122–38. CrossRef
21. Bamisile BS, Dash CK, Akutse KS, Keppanan R, Wang L. Fungal endophytes: beyond herbivore management. Front Microbiol 2018;9:544. CrossRef
22. Hoffman MT, Arnold AE. Geographic locality and host identity shape fungal endophyte communities in cupressaceous trees. Mycol Res 2008;112:331–44. CrossRef
23. Zheng Y-K, Qiao XG, Miao CP, Liu K, Chen YW, Xu LH, et al. Diversity, distribution and biotechnological potential of endophytic fungi. Ann Microbiol 2016;66(2):529–42. CrossRef
24. Rashmi M. A worldwide list of endophytic fungi with notes on ecology and diversity. Mycosphere 2019;10:798–1079. CrossRef
25. Arnold AE, Maynard Z, Gilbert GS, Coley PD, Kursar TA. Are tropical fungal endophytes hyperdiverse?. Ecol Lett 2000;3(4):267–74. CrossRef
26. Banerjee D. Endophytic fungal diversity in tropical and subtropical plants. Res J Microbiol 2011;6:54–62. CrossRef
27. Nisa H, Kamili AN, Nawchoo IA, Shafi S, Shameem N, Bandh SA. Fungal endophytes as prolific source of phytochemicals and other bioactive natural products: a review. Microb Pathogen 2015;82:50–9. CrossRef
28. Majhi P, Pradhan U, Toppo A, Shukla AK. Fungal endophytes: an insight into diversity, stress tolerance, biocontrol and plant growth-promoting potentials. Curr Microbiol 2025;82(6):283. CrossRef
29. Arnold AE, Mejía LC, Kyllo D, Rojas EI, Maynard Z, Robbins N, Herre EA. Fungal endophytes limit pathogen damage in a tropical tree. Proc Natl Acad Sci 2003; 100(26):15649–54; CrossRef
30. Ren N, Wang L, You C. Diversity, community structure, and antagonism of endophytic fungi from asymptomatic and symptomatic Mongolian pine trees. J Fungi 2024;10:212. CrossRef
31. Arnold AE, Lutzoni F. Diversity and host range of foliar fungal endophytes: are tropical leaves biodiversity hotspots?. Ecology 2007;88:541–9. CrossRef
32. Suryanarayanan TS. Diversity of fungal endophytes in tropical trees. In: Pirttilä AM, Frank AC (eds.). Endophytes of forest trees: biology and applications, Springer, Dordrecht, The Netherlands, pp 67–80, 2011. CrossRef
33. Suryanarayanan T, Venkatesan G, Murali T. Endophytic fungal communities in leaves of tropical forest trees: diversity and distribution patterns. Curr Sci 2003;85: 489–93.
34. Wang Y, Guo LD. A comparative study of endophytic fungi in needles, bark, and xylem of Pinus tabulaeformis. Botany 2007;85:911–7. CrossRef
35. Gherbawy Y, Elhariry H. Endophytic fungi associated with high-altitude Juniperus trees and their antimicrobial activities. Plant Biosyst 2016;150:131–40. CrossRef
36. Zhao J, Shan T, Mou Y, Zhou L. Plant-derived bioactive compounds produced by endophytic fungi. Mini Rev Med Chem 2011;11:159–68. CrossRef
37. Venieraki A, Dimou M, Katinakis P. Endophytic fungi residing in medicinal plants have the ability to produce the same or similar pharmacologically active secondary metabolites as their hosts. Hellenic Plant Prot J 2017;10:51–66. CrossRef
38. Mahobiya D, Gupta AK. Diversity of endophytic fungi associated with some medicinal herbs and shrubs. Kavaka 2017;49:38–44.
39. Sati SC, Belwal M. Aquatic hyphomycetes as endophytes of riparian plant roots. Mycologia 2005;97:45–9. CrossRef
40. Govinda Rajulu M. Endophytic fungi of orchids of Arunachal Pradesh, north eastern India. Curr Res Environ Appl Mycol 2016;6:293–9. CrossRef
41. Rasmussen HN. Recent developments in the study of orchid mycorrhiza. Plant Soil 2002;244:149–63. CrossRef
42. Ma X, Kang J, Nontachaiyapoom S, Wen T, Hyde KD. Non-mycorrhizal endophytic fungi from orchids. Curr Sci 2015;109: 72–87.
43. Gezgin Y, Eltem R. Diversity of endophytic fungi from various Aegean and Mediterranean orchids (saleps). Turk J Bot 2009;33:439–45. CrossRef
44. Singh SK, Strobel GA, Knighton B, Geary B, Sears J, Ezra D. An endophytic Phomopsis sp. possessing bioactivity and fuel potential with its volatile organic compounds. Microbial Ecol 2011;61:729–39. CrossRef
45. Ratnaweera PB, Williams DE, De Silva ED, Wijesundera RLC, Dalisay DS, Andersen RJ. Helvolic acid, an antibacterial nortriterpenoid from a fungal endophyte, Xylaria sp. of orchid Anoectochilus setaceus endemic to Sri Lanka. Mycology 2014;5:23–8. CrossRef
46. Sudheep NM, Sridhar KR. Non-mycorrhizal fungal endophytes in two orchids of Kaiga forest (Western Ghats), India. J For Res 2012;23:453–60. CrossRef
47. Sandberg DC, Battista LJ, Arnold AE. Fungal endophytes of aquatic macrophytes: diverse host-generalists characterized by tissue preferences and geographic structure. Microb Ecol 2014;67:735–47. CrossRef
48. Sakayaroj J, Preedanon S, Phongpaichit S, Buatong J, Chaowalit P, Rukachaisirikul V. Diversity of endophytic and marine-derived fungi associated with marine plants and animals. In: Jones EBG, Pang KL (eds.). Marine fungi and fungal-like organisms. Walter de Gruyter, Berlin, Germany, pp 291–328, 2012. CrossRef
49. Lobo M, Sridhar KR. Endophytic fungal assemblage of two halophytes from west coast mangrove habitats, India. Czech Mycol. 2003;55:241–251. CrossRef
50. Anita D, Sridhar K, Bhat R. Diversity of fungi associated with mangrove legume Sesbania bispinosa (Jacq.) W. Wight (Fabaceae). Livest Res Rural Dev 2009;21:5.
51. Shreelalitha SJ, Sridhar KR. Endophytic fungi of wild legume Sesbania bispinosa in coastal sand dunes and mangroves of the Southwest coast of India. J For Res 2015;26:1003–11. CrossRef
52. Singh VK, Dwivedy AK, Singh A, Asawa S, Dwivedi A, Dubey NK. Fungal endophytes from seaweeds: an overview. In: Patra J, Das G, Shin HS (eds.). Microbial biotechnology: volume 2 application in food and pharmacology, Springer, Singapore, p 483, 2018. CrossRef
53. Suryanarayanan T. Fungal endosymbionts of seaweeds. In: Raghukumar C (ed.). Biology of marine fungi, progress in molecular and subcellular biology, vol 53. Springer, Berlin, Germany, pp 53–69, 2011. CrossRef
54. Devarajan P, Suryanarayanan T. Endophytic fungi associated with the tropical seagrass Halophila ovalis (Hydrocharitaceae). Ind J Mar Sci 2002;31:73–4.
55. Venkatachalam A, Thirunavukkarasu N, Suryanarayanan TS. Distribution and diversity of endophytes in seagrasses. Fungal Ecol 2015;13:60–5. CrossRef
56. Alva P, McKenzie E, Pointing S, Pena-Muralla R, Hyde K. Do seagrasses harbour endobiotes?. In: Hyde KD (ed.). Fungi in marine environments, Fungal Divers Press, Hong Kong, China, pp 167–78, 2002.
57. Singh A, Singh DK, Kharwar RN, White JF, Gond SK. Fungal endophytes as efficient sources of plant-derived bioactive compounds and their prospective applications in natural product drug discovery: insights, avenues, and challenges. Microorganisms 2021;9(1):197. CrossRef
58. Ancheeva E, Daletos G, Proksch P. Bioactive secondary metabolites from endophytic fungi. Curr Med Chem 2020;27:1836–54. CrossRef
59. Eyberger AL, Dondapati R, Porter JR. Endophyte fungal isolates from Podophyllum peltatum produce podophyllotoxin. J Nat Prod 2006;69(8):1121–4. CrossRef
60. Meshram V, Kapoor N, Dwibedi V, Srivastava A, Saxena S. Extracellular resveratrol producing endophytic fungus, Quambalaria cyanescens. South Afr J Bot 2022;146:409–16. CrossRef
61. Meshram V, Saxena S, Paul K. Xylarinase: a novel clot busting enzyme from an endophytic fungus Xylaria curta. J Enzyme Inhib Med Chem 2016;31:1502–11. CrossRef
62. Manganyi MC, Ateba CN. Untapped potentials of endophytic fungi: a review of novel bioactive compounds with biological applications. Microorganisms 2020;8:1934. CrossRef
63. Hashem AH, Attia MS, Kandil EK, Fawzi MM, Abdelrahman AS, Khader MS, et al. Bioactive compounds and biomedical applications of endophytic fungi: a recent review. Microb Cell Fac 2023;22:107. CrossRef
64. Mayer AMS, Guerrero AJ, Rodríguez AD, Taglialatela-Scafati O, Nakamura F, Fusetani N. Marine pharmacology in 2014–2015: marine compounds with antibacterial, antidiabetic, antifungal, anti-inflammatory, antiprotozoal, antituberculosis, antiviral, and anthelmintic activities; affecting the immune and nervous systems, and other miscellaneous mechanisms of action. Mar Drugs 2019;18:5. CrossRef
65. Wijeratne EMK, He H, Franzblau SG, Hoffman AM, Gunatilaka AAL. Phomapyrrolidones A–C, antitubercular alkaloids from the endophytic fungus Phoma sp. NRRL 46751. J Nat Prod 2013;76:1860–5. CrossRef
66. Tan Y, Guo Z, Zhu M, Shi J, Li W, Jiao R, et al. Anti-inflammatory spirobisnaphthalene natural products from a plant-derived endophytic fungus Edenia gomezpompae. Chin Chem Lett 2020;31:1406–9. CrossRef
67. Pina JRS, Silva-Silva JV, Carvalho JM, Bitencourt HR, Watanabe LA, Fernandes JMP, et al. Antiprotozoal and antibacterial activity of ravenelin, a xanthone isolated from the endophytic fungus Exserohilum rostratum. Molecules 2021;26:3339. CrossRef
68. Zhang P, Yuan XL, Du YM, Zhang HB, Shen GM, Zhang ZF, et al. Angularly prenylated indole alkaloids with antimicrobial and insecticidal activities from an endophytic fungus Fusarium sambucinum TE-6L. J Agric Food Chem 2019;67:11994–2001. CrossRef
69. Hawas UW, Abou El-kassem LT. Anticancer and antiviral diketopiperazine produced by the Red Sea endophytic fungus Penicillium chrysogenum. Lett Org Chem 2019;16:409–14. CrossRef
70. Rauf M, Ur-Rahman A, Arif M, Gul H, Ud-Din A, Hamayun M, et al. Immunomodulatory molecular mechanisms of Luffa cylindrica for downy mildews resistance induced by growth-promoting endophytic fungi. J Fungi 2022;8:689. CrossRef
71. Zhao J, Mou Y, Shan T, Li Y, Zhou L, Wang M, et al. Antimicrobial metabolites from the endophytic fungus Pichia guilliermondii isolated from Paris polyphylla var. yunnanensis. Molecules 2010;15(11):7961–70. CrossRef
72. Zhao J, Li C, Wang W, Zhao C, Luo M, Mu F, et al. Hypocrea lixii, novel endophytic fungi producing anticancer agent cajanol, isolated from pigeon pea (Cajanus cajan L. Millsp.). J Appl Microbiol 2013;115:102–13. CrossRef
73. Huang JX, Zhang J, Zhang XR, Zhang K, Zhang X, He XR. Mucor fragilis as a novel source of the key pharmaceutical agents podophyllotoxin and kaempferol. Pharm Biol 2014;52:1237–43. CrossRef
74. Deshmukh SK, Mishra PD, Kulkarni-Almeida A, Verekar S, Sahoo MR, Periyasamy G, et al. Anti-inflammatory and anticancer activity of ergoflavin isolated from an endophytic fungus. Chem Biodivers 2009;6:784–9. CrossRef
75. Sadananda T, Govindappa M, Vinay Dutt G, Bhat B, Baishya P, Chandrappa C. Isolation and characterization of antiviral and ribosome inactivating protein from the endophytic fungi Alternaria sp from Viscum album using MADLI-TOF-MS and their antibacterial activity. Drug Invent Today. 2014;6(2):105–112.
76. Zhang H, Ying C, Bai X. Advancement in endophytic microbes from medicinal plants. Int J Pharma Sci Res 2014;5:1589.
77. Song XQ, Zhang X, Han QJ, Li XB, Li G, Li RJ, et al. Xanthone derivatives from Aspergillus sydowii, an endophytic fungus from the liverwort Scapania ciliata S. Lac and their immunosuppressive activities. Phytochem Lett 2013;6:318–21. CrossRef
78. Turbyville TJ, Wijeratne EMK, Liu MX, Burns AM, Seliga CJ, Luevano LA, et al. Search for Hsp90 inhibitors with potential anticancer activity: isolation and SAR studies of radicicol and monocillin I from two plant-associated fungi of the Sonoran desert. J Nat Prod 2006;69:178–84. CrossRef
79. Waqas M, Khan AL, Kamran M, Hamayun M, Kang SM, Kim YH, Lee IJ. Endophytic fungi produce gibberellins and indoleacetic acid and promotes host-plant growth during stress. Molecules. 2012;17(9):10754–10773. CrossRef
80. Lo Presti L, Lanver D, Schweizer G, Tanaka S, Liang L, Tollot M, et al. Fungal effectors and plant susceptibility. Ann Rev Plant Biol 2015;66:513–45. CrossRef
81. Elumalai P, Gao X, Parthipan P, Luo J, Cui J. Agrochemical pollution: a serious threat to environmental health. Current Opinion in Environmental Science & Health. 2025;43:100597. CrossRef
82. Bamisile BS, Akutse KS, Siddiqui JA, Xu Y. Model application of entomopathogenic fungi as alternatives to chemical pesticides: prospects, challenges, and insights for next-generation sustainable agriculture. Front Plant Sci 2021;12:741804. CrossRef
83. Sravani B, Shirisha T, Blesseena A, Narute T. Fungal endophytes: classification and functional role in sustainable agriculture. Krishi Sci eMagazine Agric Sci 2020;1:24–7.
84. Auer S, Ludwig-Müller J. Biological control of clubroot (Plasmodiophora brassicae) by the endophytic fungus Acremonium alternatum. J Endocytobiosis Cell Res 2015;26:43–9.
85. Ek-Ramos MJ, Zhou W, Valencia CU, Antwi JB, Kalns LL, Morgan GD, et al. Spatial and temporal variation in fungal endophyte communities isolated from cultivated cotton (Gossypium hirsutum). PLoS One 2013;8:e66049. CrossRef
86. Amatuzzi R, Cardoso N, Poltronieri A, Poitevin C, Dalzoto P, Zawadeneak M, et al. Potential of endophytic fungi as biocontrol agents of Duponchelia fovealis (Zeller) (Lepidoptera: crambidae). Braz J Biol 2017;78:429–35. CrossRef
87. Han LR, Wang ZH, Zhang HJ, Xue LS, Feng JT, Zhang X. Isolation of endophytic fungi from Tripterygium wilfordii and their insecticidal activities. Afr J Microbiol Res 2013;7:771–6.
88. El-Sayed ASA, Moustafa AH, Hussein HA, El-Sheikh AA, El-Shafey SN, Fathy NAM, et al. Potential insecticidal activity of Sarocladium strictum, an endophyte of Cynanchum acutum, against Spodoptera littoralis, a polyphagous insect pest. Biocatal Agric Biotechnol 2020;24:101524. CrossRef
89. Chen D, Zhang P, Liu T, Wang XF, Li ZX, Li W, et al. Insecticidal activities of chloramphenicol derivatives isolated from a marine alga-derived endophytic fungus, Acremonium vitellinum, against the cotton bollworm, Helicoverpa armigera (Hübner) (Lepidoptera: noctuidae). Molecules 2018;23:2995. CrossRef
90. Pascholati S, De Souza V, Cardoso Filho J. Trichoderma: uso na agricultura. In: Meyer MC, Mazaro SM, Silva JC da. Embrapa Soja-Livro científico (ALICE), Embrapa, Brazil, vol. 7, p 235, 2019.
91. Sharon E, Chet I, Viterbo A, Bar-Eyal M, Nagan H, Samuels GJ, et al. Parasitism of Trichoderma on Meloidogyne javanica and role of the gelatinous matrix. Eur J Plant Pathol 2007;118:247–58. CrossRef
92. Das MM, Herrera RR, Haridas M, Sabu A. Purpureocillium lilacinum: a promising bionematicide for sustainable agriculture. In: Rojas R, Ávila GCGM, Contreras JAV, Aguilar CN (eds.). Biocontrol systems and plant physiology in modern agriculture, Apple Academic Press, Palm Bay, FL, pp 61–91, 2022. CrossRef
93. Toksöz S, Oksal E, Akça I. Effect of entomopathogenic fungus, Purpureocillium lilacinum (syn: paecilomyces lilacinus) on Blatta orientalis and Shelfordella tartara under laboratory conditions. Mun Ent Zool 2019;14:259–64.
94. Kamel RA, Abdel-Razek AS, Hamed A, Ibrahim RR, Stammler HG, Frese M, et al. Isoshamixanthone: a new pyrano xanthone from endophytic Aspergillus sp. ASCLA and absolute configuration of epiisoshamixanthone. Nat Prod Res 2020;34:1080–90. CrossRef
95. Zhao T, Xu LL, Zhang Y, Lin ZH, Xia T, Yang DF, et al. Three new α-pyrone derivatives from the plant endophytic fungus Penicillium ochrochloronthe and their antibacterial, antifungal, and cytotoxic activities. J Asian Nat Prod Res 2019;21:851–8. CrossRef
96. Ramos HP, Braun GH, Pupo MT, Said S. Antimicrobial activity from endophytic fungi Arthrinium state of Apiospora montagnei Sacc. and Papulaspora immersa. Braz Arch Biol Technol 2010;53:629–32. CrossRef
97. Hussein ME, Mohamed OG, El-Fishawy AM, El-Askary HI, El-Senousy AS, El-Beih AA, et al. Identification of antibacterial metabolites from endophytic fungus Aspergillus fumigatus, isolated from Albizia lucidior leaves (Fabaceae), utilizing metabolomic and molecular docking techniques. Molecules 2022;27:1117. CrossRef
98. Sharaf MH, Abdelaziz AM, Kalaba MH, Radwan AA, Hashem AH. Antimicrobial, antioxidant, cytotoxic activities and phytochemical analysis of fungal endophytes isolated from Ocimum basilicum. Appl Biochem Biotechnol 2022;194:1271–89. CrossRef
99. Arivudainambi USE, Anand TD, Shanmugaiah V, Karunakaran C, Rajendran A. Novel bioactive metabolites producing endophytic fungus Colletotrichum gloeosporioides against multidrug-resistant Staphylococcus aureus. FEMS Immunol Med Microbiol 2011;61:340–5. CrossRef
100. Chandra H, Kumari P, Prasad R, Chandra Gupta S, Yadav S. Antioxidant and antimicrobial activity displayed by a fungal endophyte Alternaria alternata isolated from Picrorhiza kurroa from Garhwal Himalayas, India. Biocatal Agric Biotechnol 2021;33:101955. CrossRef
101. Maliehe TS, Mbambo M, Nqotheni MI, Senzo NS, Shandu JSE. Antibacterial effect and mode of action of secondary metabolites from fungal endophyte associated with Aloe ferox Mill. Microbiol Res 2022;13:90–101. CrossRef
102. Kumari P, Singh A, Singh DK, Sharma VK, Kumar J, Gupta VK, et al. Isolation and purification of bioactive metabolites from an endophytic fungus Penicillium citrinum of Azadirachta indica. South Afr J Bot 2021;139:449–57. CrossRef
103. Elkhouly HI, Hamed AA, El Hosainy AM, Ghareeb MA, Sidkey NM. Bioactive secondary metabolite from endophytic Aspergillus tubenginses ASH4 isolated from Hyoscyamus muticus: antimicrobial, antibiofilm, antioxidant and anticancer activity. Pharmacog J 2021;13:434–42. CrossRef
104. Nurunnabi TR, Sabrin F, Sharif DI, Nahar L, Sohrab MH, Sarker SD, et al. Antimicrobial activity of endophytic fungi isolated from the mangrove plant Sonneratia apetala (Buch.-Ham) from the Sundarbans mangrove forest. Adv Trad Med 2020;20:419–25. CrossRef
105. Wu H, Yan Z, Deng Y, Wu Z, Xu X, Li X, et al. Endophytic fungi from the root tubers of medicinal plant Stephania dielsiana and their antimicrobial activity. Acta Ecol Sin 2020;40:383–7. CrossRef
106. Ding Z, Tao T, Wang L, Zhao Y, Huang H, Zhang D, et al. Bioprospecting of novel and bioactive metabolites from endophytic fungi isolated from rubber tree Ficus elastica leaves. J Microbiol Biotechnol 2019;29:731-8. CrossRef
107. Nischitha R, Shivanna MB. Metabolite fingerprinting, in vitro antimicrobial and antioxidant activities and in-silico docking in Alloteropsis cimicina and its endophytic fungus Penicillium pinophilum. Mol Biol Rep 2021;48:4021–37. CrossRef
108. Supaphon P, Preedanon S. Evaluation of in vitro alpha-glucosidase inhibitory, antimicrobial, and cytotoxic activities of secondary metabolites from the endophytic fungus, Nigrospora sphaerica, isolated from Helianthus annuus. Ann Microbiol 2019;69:1397–406. CrossRef
109. Yasser MM, Marzouk MA, El-Shafey NM, Shaban SA. Diversity and antimicrobial activity of endophytic fungi from the medicinal plant Pelargonium graveolens (geranium) in Middle Egypt. Jordan J Biol Sci 2020;13:197–205.
110. Tanapichatsakul C, Khruengsai S, Monggoot S, Pripdeevech P. Production of eugenol from fungal endophytes Neopestalotiopsis sp. and Diaporthe sp. isolated from Cinnamomum loureiroi leaves. PeerJ 2019;7:e6427. CrossRef
111. Han M, Qin D, Ye T, Yan X, Wang J, Duan X, et al. An endophytic fungus from Trichoderma harzianum SWUKD3.1610 that produces nigranoic acid and its analogues. Nat Prod Res 2019;33:2079–87.
112. Moussa AY, Mostafa NM, Singab ANB. Pulchranin A: first report of isolation from an endophytic fungus and its inhibitory activity on cyclin dependent kinases. Nat Prod Res 2020;34:2715–22.
113. Schulz B, Haas S, Junker C, Andrée N, Schobert M. Fungal endophytes are involved in multiple balanced antagonisms. Curr Sci 2015;109:39-45.
114. Chitnis VR, Suryanarayanan TS, Nataraja KN, Prasad SR, Oelmüller R, Shaanker RU. Fungal endophyte-mediated crop improvement: the way ahead. Front Plant Sci 2020;11:561007.
115. Domka AM, Rozpa?dek P, Turnau K. Are fungal endophytes merely mycorrhizal copycats? The role of fungal endophytes in the adaptation of plants to metal toxicity. Front Microbiol 2019;10:371.
116. Tabbasum I, Ali A, Shafique U, Bibi I, Khalid B, Ijaz N, et al. Role of endophytic fungal species in plant growth promotion and in sustainable agricultural productions: a review. J Microbiol Mol Genet 2022;3:1–21.
117. Khan AL, Hussain J, Al-Harrasi A, Al-Rawahi A, Lee IJ. Endophytic fungi: resource for gibberellins and crop abiotic stress resistance. Crit Rev Biotechnol 2015;35:62–74.
118. Jaroszuk-?cise? J, Kurek E, Trytek M. Efficiency of indoleacetic acid, gibberellic acid and ethylene synthesized in vitro by Fusarium culmorum strains with different effects on cereal growth. Biologia 2014;69:281–92.
119. Bömke C, Tudzynski B. Diversity, regulation, and evolution of the gibberellin biosynthetic pathway in fungi compared to plants and bacteria. Phytochemistry 2009;70:1876–93.
120. Baron NC, Souza Pollo AD, Rigobelo EC. Purpureocillium lilacinum and Metarhizium marquandii as plant growth-promoting fungi. PeerJ 2020;8:e9005.
121. Lubna, Asaf S, Hamayun M, Gul H, Lee IJ, Hussain A. Aspergillus niger CSR3 regulates plant endogenous hormones and secondary metabolites by producing gibberellins and indoleacetic acid. J Plant Interact 2018;13:100–11.
122. Sarkar S, Dey A, Kumar V, Batiha GES, El-Esawi MA, Tomczyk M, et al. Fungal endophyte: an interactive endosymbiont with the capability of modulating host physiology in myriad ways. Front Plant Sci 2021;12:701800.
123. Tandon A, Fatima T, Shukla D, Tripathi P, Srivastava S, Singh PC. Phosphate solubilization by Trichoderma koningiopsis (NBRI-PR5) under abiotic stress conditions. J King Saud Univ Sci 2020;32:791–8.
124. Zhang S, Gan Y, Xu B. Mechanisms of the IAA and ACC-deaminase producing strain of Trichoderma longibrachiatum T6 in enhancing wheat seedling tolerance to NaCl stress. BMC Plant Biol 2019;19:1–8.
125. Hassan SED. Plant growth-promoting activities for bacterial and fungal endophytes isolated from medicinal plant of Teucrium polium L. J Adv Res 2017;8:687–95.
126. Airin AA, Arafat MI, Begum RA, Islam MR, Seraj ZI. Plant growth-promoting endophytic fungi of the wild halophytic rice Oryza coarctata. Ann Microbiol 2023;73:36.
127. Suebrasri T, Harada H, Jogloy S, Ekprasert J, Boonlue S. Auxin-producing fungal endophytes promote growth of sunchoke. Rhizosphere 2020;16:100271.
128. Lledó S, Rodrigo S, Poblaciones MJ, Santamaria O. Biomass yield, nutritive value and accumulation of minerals in Trifolium subterraneum L. as affected by fungal endophytes. Plant Soil 2016;405:197–210.
129. García-Latorre C, Rodrigo S, Marin-Felix Y, Stadler M, Santamaria O. Plant-growth promoting activity of three fungal endophytes isolated from plants living in dehesas and their effect on Lolium multiflorum. Scientific Rep 2023;13:7354.
130. Adedayo AA, Babalola OO. Fungi that promote plant growth in the rhizosphere boost crop growth. J Fungi 2023;9:239.
131. Omomowo IO, Adedayo AA, Omomowo OI. Biocontrol potential of rhizospheric fungi from Moringa oleifera, their phytochemicals and secondary metabolite assessment against spoilage fungi of sweet orange (Citrus sinensis). Asian J Appl Sci 2020;8:35-48.
132. Attia MS, Abdelaziz AM, Al-Askar AA, Arishi AA, Abdelhakim AM, Hashem AH. Plant growth-promoting fungi as biocontrol tool against fusarium wilt disease of tomato plant. J Fungi 2022;8:775.
133. Kuzin A, Solovchenko A, Stepantsova L, Pugachev G. Soil fertility management in apple orchard with microbial biofertilizers. In E3S Web Conf. 2020;222:03020.
134. Cantabella D, Dolcet-Sanjuan R, Casanovas M, Solsona C, Torres R, Teixidó N. Inoculation of in vitro cultures with rhizosphere microorganisms improve plant development and acclimatization during immature embryo rescue in nectarine and pear breeding programs. Sci Hortic 2020;273:109643.
135. Syamsia SS, Abubakar AI, Amanda APF, Noerfitryani NN, Iradhatullah IR, Henry HK, et al. Combination on endophytic fungal as the plant growth-promoting fungi (PGPF) on cucumber (Cucumis sativus). Biodiversitas 2021;22:1194–202.
136. Pandit MA, Kumar J, Gulati S, Bhandari N, Mehta P, Katyal R, et al. Major biological control strategies for plant pathogens. Pathogens 2022;11:273.
137. Hossain MdM, Sultana F, Islam S. Plant Growth-Promoting Fungi (PGPF): Phytostimulation and Induced Systemic Resistance. Plant-Microbe Interactions in Agro-Ecological Perspectives. 2017;135–91.
138. Chatterjee S, Ghosh R, Mandal NC. Production of bioactive compounds with bactericidal and antioxidant potential by endophytic fungus Alternaria alternata AE1 isolated from Azadirachta indica A. Juss. PLoS One 2019;14:e0214744.
139. Pai G, Chandra M. Antimicrobial activity of endophytic fungi isolated from ethnomedicinal plant Phyllanthus reticulatus poir. Int J Eng Sci Invention 2018;7:40–6.
140. Govindappa M, Hemmanur KC, Nithin S, Poojari CC, Bhat G, Channabasava K. In vitro anti-HIV activity of partially purified coumarin (s) isolated from fungal endophyte, Alternaria species of Calophyllum inophyllum. Pharmacol Pharm 2015;6:321. CrossRef
141. Gao Y, Wang L, Kalscheuer R, Liu Z, Proksch P. Antifungal polyketide derivatives from the endophytic fungus Aplosporella javeedii. Bioorg Med Chem 2020;28:115456. CrossRef
142. Pinheiro EAA, Carvalho JM, Dos Santos DCP, Feitosa ADO, Marinho PSB, Guilhon GMSP, et al. Antibacterial activity of alkaloids produced by endophytic fungus Aspergillus sp. EJC08 isolated from medical plant Bauhinia guianensis. Nat Prod Res 2013;27:1633–8. CrossRef
143. Zihad SMNK, Hasan MT, Sultana MS, Nath S, Nahar L, Rashid MA, et al. Isolation and characterization of antibacterial compounds from Aspergillus fumigatus: an endophytic fungus from a mangrove plant of the Sundarbans. Evid Based Complement Alternat Med 2022;9600079. CrossRef
144. Premjanu N, Jaynthy C, Diviya S. Antifungal activity of endophytic fungi isolated from Lannea coromandelica–an in silico approach. Int J Pharm Pharm Sci 2016;8:207–10.
145. Mishra VK, Passari AK, Chandra P, Leo VV, Kumar B, Uthandi S, et al. Determination and production of antimicrobial compounds by Aspergillus clavatonanicus strain MJ31, an endophytic fungus from Mirabilis jalapa L. using UPLC-ESI-MS/MS and TD-GC-MS analysis. PLoS One 2017;12:e0186234. CrossRef
146. Elkady WM, Raafat MM, Abdel-Aziz MM, Al-Huqail AA, Ashour ML, Fathallah N. Endophytic fungus from Opuntia ficus-indica: a source of potential bioactive antimicrobial compounds against multidrug-resistant bacteria. Plants 2022;11:1070. CrossRef
147. Techaoei S, Jirayuthcharoenkul C, Jarmkom K, Dumrongphuttidecha T, Khobjai W. Chemical evaluation and antibacterial activity of novel bioactive compounds from endophytic fungi in Nelumbo nucifera. Saudi J Biol Sci 2020;27(11):2883-9. CrossRef
148. Pansanit A, Pripdeevech P. Antibacterial secondary metabolites from an endophytic fungus, Arthrinium sp. MFLUCC16-1053 isolated from Zingiber cassumunar. Mycology 2018;9:264–72. CrossRef
149. Ding X, Liu K, Deng B, Chen W, Li W, Liu F. Isolation and characterization of endophytic fungi from Camptotheca acuminata. World J Microbiol Biotechnol 2013;29:1831–8. CrossRef
150. Hilario F, Polinário G, De Amorim MR, De Sousa Batista V, Do Nascimento Júnior NM, Araújo AR, et al. Spirocyclic lactams and curvulinic acid derivatives from the endophytic fungus Curvularia lunata and their antibacterial and antifungal activities. Fitoterapia 2020;141:104466. CrossRef
151. Nischitha R, Shivanna MB. Antimicrobial activity and metabolite profiling of endophytic fungi in Digitaria bicornis (Lam) Roem. and Schult. and Paspalidium flavidum (Retz.) A. Camus. 3 Biotech 2021;11:53. CrossRef
152. Kaaniche F, Hamed A, Abdel-Razek AS, Wibberg D, Abdissa N, El Euch IZ, et al. Bioactive secondary metabolites from new endophytic fungus Curvularia sp isolated from Rauwolfia macrophylla. PLoS One 2019;14:e0217627. CrossRef
153. Venkateswarulu N, Shameer S, Bramhachari PV, Basha SKT, Nagaraju C, Vijaya T. Isolation and characterization of plumbagin (5-hydroxyl-2-methylnaptalene-1, 4-dione) producing endophytic fungi Cladosporium delicatulum from endemic medicinal plants. Biotechnol Rep 2018;20:e00282. CrossRef
154. Yehia RS, Osman GH, Assaggaf H, Salem R, Mohamed MSM. Isolation of potential antimicrobial metabolites from endophytic fungus Cladosporium cladosporioides from endemic plant Zygophyllum mandavillei. South Afr J Bot 2020;134:296–302. CrossRef
155. Lu H, Zou WX, Meng JC, Hu J, Tan RX. New bioactive metabolites produced by Colletotrichum sp., an endophytic fungus in Artemisia annua. Plant Sci 2000;151:67–73. CrossRef
156. Wang WX, Kusari S, Laatsch H, Golz C, Kusari P, Strohmann C, et al. Antibacterial azaphilones from an endophytic fungus, Colletotrichum sp. BS4. J Nat Prod 2016;79:704–10. CrossRef
157. Hussain H, Root N, Jabeen F, Al-Harrasi A, Al-Rawahi A, Ahmad M, et al. Seimatoric acid and collotonioic acid: two new compounds from the endophytic fungi, Seimatosporium sp. and Colletotrichum sp. Chin Chem Lett 2014;25:1577–9. CrossRef
158. Chen C, Zhu H, Wang J, Yang J, Li XN, Wang J, et al. Armochaetoglobins K–R, Anti-HIV pyrrole-based cytochalasans from Chaetomium globosum TW1-1. Eur J Org Chem 2015;2015:3086–94. CrossRef
159. Sebastianes FLS, Cabedo N, Aouad NE, Valente AMMP, Lacava PT, Azevedo JL, et al. 3-Hydroxypropionic acid as an antibacterial agent from endophytic fungi Diaporthe phaseolorum. Curr Microbiol 2012;65:622–32. CrossRef
160. Guo L, Niu S, Chen S, Liu L. Diaporone A, a new antibacterial secondary metabolite from the plant endophytic fungus Diaporthe sp. J Antibiot 2020;73:116–9. CrossRef
161. Zhang G, Sun S, Zhu T, Lin Z, Gu J, Li D, et al. Antiviral isoindolone derivatives from an endophytic fungus Emericella sp. associated with Aegiceras corniculatum. Phytochemistry 2011;72:1436–42. CrossRef
162. Li G, Kusari S, Lamshöft M, Schüffler A, Laatsch H, Spiteller M. Antibacterial secondary metabolites from an endophytic fungus, Eupenicillium sp. LG41. J Nat Prod 2014;77:2335–41. CrossRef
163. Goutam J, Kharwar R, Tiwari V, Mishra A, Singh S. Isolation and identification of antibacterial compounds isolated from endophytic fungus Emericella qaudrilineata. Nat Prod Chem Res 2016;4:2. CrossRef
164. Xian PJ, Liu SZ, Wang WJ, Yang SX, Feng Z, Yang XL. Undescribed specialised metabolites from the endophytic fungus Emericella sp. XL029 and their antimicrobial activities. Phytochemistry 2022;202:113303. CrossRef
165. Dzoyem JP, Melong R, Tsamo AT, Maffo T, Kapche DGWF, Ngadjui BT, et al. Cytotoxicity, antioxidant and antibacterial activity of four compounds produced by an endophytic fungus Epicoccum nigrum associated with Entada abyssinica. Rev Bras Farmacogn 2017;27:251–3. CrossRef
166. Prabukumar S, Rajkuberan C, Ravindran K, Sivaramakrishnan S. Isolation and characterization of endophytic fungi from medicinal plant Crescentia cujete L. and their antibacterial, antioxidant and anticancer properties. Int J Pharm Pharm Sci 2015;7:316–21.
167. Bungtongdee N, Sopalun K, Laosripaiboon W, Iamtham S. The chemical composition, antifungal, antioxidant and antimutagenicity properties of bioactive compounds from fungal endophytes associated with Thai orchids. J Phytopathol 2019;167:56–64. CrossRef
168. Zhao J. Antimicrobial metabolites from the endophytic fungus Gliomastix murorum Ppf8 associated with the medicinal plant Paris polyphylla var. yunnanensis. J Med Plants Res 2012;6:2100–4. CrossRef
169. Liang HQ, Zhang DW, Guo SX, Yu J. Two new tetracyclic triterpenoids from the endophytic fungus Hypoxylon sp. 6269. J Asian Nat Prod Res 2018;20:951–6. CrossRef
170. Meng X, Mao Z, Lou J, Xu L, Zhong L, Peng Y, et al. Benzopyranones from the endophytic fungus Hyalodendriella sp. Ponicetia deflexa and their bioactivities. Molecules 2012;17:11303–14. CrossRef
171. Sumarah MW, Kesting JR, Sørensen D, Miller JD. Antifungal metabolites from fungal endophytes of Pinus strobus. Phytochemistry 2011;72:1833–7. CrossRef
172. Mcmullin DR, Green BD, Miller JD. Antifungal sesquiterpenoids and macrolides from an endophytic Lophodermium species of Pinus strobus. Phytochem Lett 2015;14:148–52. CrossRef
173. Hussain H, Root N, Jabeen F, Al-Harrasi A, Ahmad M, Mabood F, et al. Microsphaerol and seimatorone: two new compounds isolated from the endophytic fungi, Microsphaeropsis sp. and Seimatosporium sp. Chem Biodivers 2015;12:289–94. CrossRef
174. Strobel G. Muscodor albus and its biological promise. J Ind Microbiol Biotechnol 2006;33:514. CrossRef
175. Strobel G. The emergence of endophytic microbes and their biological promise. J Fungi 2018;4:57. CrossRef
176. Akpotu M, Eze P, Ajaghaku D, Okoye F, Esimone C. Antimicrobial activity of endophytic fungi isolated from Catharanthus roseus and Euphorbia hirta. Planta Med 2015;81:145. CrossRef
177. Zhang SP, Huang R, Li FF, Wei HX, Fang XW, Xie XS, et al. Antiviral anthraquinones and azaphilones produced by an endophytic fungus Nigrospora sp. from Aconitum carmichaeli. Fitoterapia 2016;112:85–9. CrossRef
178. Dos Santos IP, da Silva LC, da Silva MV, de Araújo JM, Cavalcanti Mda S, Lima VL. Antibacterial activity of endophytic fungi from leaves of Indigofera suffruticosa Miller (Fabaceae). Front Microbiol 2015;6:350. CrossRef
179. Silva GH, Teles HL, Zanardi LM, Young MC, Eberlin MN, Hadad R, et al. Cadinane sesquiterpenoids of Phomopsis cassiae, an endophytic fungus associated with Cassia spectabilis (Leguminosae). Phytochemistry 2006;67(17):1964–9. CrossRef
180. Hoffman AM, Mayer SG, Strobel GA, Hess WM, Sovocool GW, Grange AH, et al. Purification, identification and activity of phomodione, a furandione from an endophytic Phoma species. Phytochemistry 2008;69:1049–56. CrossRef
181. Sharma D, Pramanik A, Agrawal PK. Evaluation of bioactive secondary metabolites from endophytic fungus Pestalotiopsis neglecta BAB-5510 isolated from leaves of Cupressus torulosa D. Don. 3 Biotech 2016;6:210. CrossRef