
1. INTRODUCTION
Citrus limon (L.) Osbeck is an evergreen species under the Rutaceae family with more than 30 different types of lemons existing throughout the world, some of which are indigenous to certain specific regions [1,2]. Citrus limon “Assam lemon” (AL) as such is an important and indigenous cultivar of Assam [3,4]. AL is locally known as ‘Kaji Nemu’ in Assam and is widely used as a table fruit due to its seedless character [5]. AL has a distinct aroma, flavor, and fruit characteristics that distinguish it from the other lemon cultivars [6,7].
AL is abundant in several vital physio-biochemical substances, which are beneficial to human health and aid in the prevention of a variety of diseases [5,8]. The physiological and biological changes that take place during fruit growth, development, and maturity are largely responsible for the changes in physio-biochemical and storage life of fruits [9]. It was reported that AL fruits are typically sold in the markets for 45 to 60 days after fruit setting (DAF). Picking fruit at the wrong stage is known to lower nutritional and flavor quality [10].
As physio-biochemical concentration fluctuates at different stages of fruit development (DSFD), the food and pharmaceutical industries choose fruits from different stages depending on the need [11]. Though few studies on AL physio-biochemical analysis at DSFD have been reported, a lack of in-depth analysis from its immature (7 DAF) to its fully mature stage (150 DAF) was observed. In addition, physio-biochemical differentiation in peel (PL) and pulp (PP) in fruits of AL at DSFD was found to be lacking. Furthermore, no reports were found on parameters related to pectin purity and the degree of pectin esterification in AL fruit PL and PP, which is a crucial factor for selection in various food and pharmaceutical industries. In the current study, these knowledge gaps on physio-biochemical variation analysis for harvesting and selection of quality fruits were addressed.
Storage temperature is a critical factor in postharvest handling and storage, as it directly affects the physio-biochemical processes in fruits [12]. Improper storage conditions also lead to weight loss, textural changes, color deterioration, etc., resulting in reduced market value and consumer acceptance of AL [13]. Therefore, studying how varying storage temperatures affect AL fruit is essential for identifying optimal storage conditions [14].
This study endeavors to gain more insights into physical and physio-biochemical variations in both PL and PP of Assam lemon fruit (ALF) during DSFD, along with storage at room temperature (SRT) and cold temperatures (SCT). This research will be valuable for determining optimal harvest times, methods for prolonging shelf life, and maintaining fruit quality. By exploring these, valuable insights can be obtained for enhancing postharvest practices, storage techniques, and decision-making for producers, distributors, and consumers.
2. MATERIALS AND METHODS
2.1. Plant Materials
For the present study, 48 ALF were collected from trees located at Assam Agricultural University-Horticulture Research Station (AAU-HRS), Kahikuchi (Latitude - 26.107098, Longitude- 91.610368). Before the fruit set, 96 developing flowers were tagged, and 3 fruits per stage/condition were collected at different DAF set, including 7, 15, 30, 45, 60, 90, 120, and 150 DAF (Fig. 1) for physical and physio-biochemical investigation.
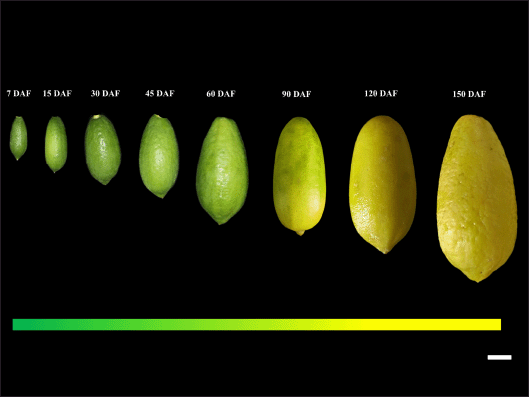 | Figure 1. ALFs at different stages of their development (scale bar-0.75 cm). [Click here to view] |
For the postharvest study, ALF were harvested at 150 DAF and (SRT; 27°C ± 2°C) and (SCT; 4°C) for a duration of 28 days. The stored samples were analyzed at specific intervals, namely at 7 days after storage (DAS), 15, 21, and 28 DAS.
2.2. Physical Characteristics Analysis
The different physical characteristics of ALF were studied including fruit weight (g), fruit length (cm), fruit breadth (cm), fruit color, specific gravity, PL weight (g), PP weight (g), fruit PP ratio, rind thickness of PL (mm), flavedo thickness of PL (mm), albedo thickness of PL (mm), pith diameter of fruit (mm), and pith to albedo length (LPA) (mm). During this investigation, the fruit weight, PL weight, and PP weight were measured using an electronic balance. Further, fruit length, fruit breadth, specific gravity, fruit rind thickness of PL, flavedo thickness of PL, albedo thickness of PL, and LPA were studied using a digital vernier caliper, additionally with the specific gravity, which was calculated as weight per unit volume of ALF.
2.3. Physio-Biochemical Analysis
The different fruit quality parameters of DSFD were investigated including pH, % juice content (% JC), total soluble solids (TSS) (°Brix), citric acid (g/ml), ascorbic acid (mg/ml), TSS/titratable acidity (TA), total sugar (TS) (μg/ml), reducing sugar (RS) (μg/ml), carotenoid concentration (mg/g), chlorophyll content (μg/g), pectin content (PC) (PL and PP), equivalent weight (EW) content (PL and PP), methoxyl content (MeOC) (PL and PP), anhydrouronic acid (AUA) content (PL and PP), and degree of esterification (DE) content (PL and PP). The physio-biochemical analyses were performed according to our previously published protocols [15]. The units for the biochemical parameters in this study were selected in accordance with the analytical methods used, aligning with commonly accepted reporting standards in biochemical and food analysis studies.
2.4. Estimation of Soil Nutrient
Samples of soil were collected at DSFD from AAU-HRS, Kahikuchi was examined using kits for testing soil (K054 - 1KT and K095L - 1KT, Himedia) to evaluate the amount of micro nutrients (Cu, Zn, B, Mn, Fe, and Mo) and macro nutrients (pH, OC, PO4³-, K, NH3-N, and NO3-N) present in the soil from the site of sample collection. As these kit-based methods yield results in value ranges, they are considered semi-quantitative and indicative, providing approximate rather than precise measurements of soil nutrient concentrations.
2.5. Statistical Analysis
For statistical analysis, numerical data were generated from morphological characters and physio-biochemical attributes assessed during the present investigation. The data were analyzed separately for two experimental sets: fruit developmental stages (7–150 DAF) and storage conditions (SRT- 7 DAS- 28 DAS, SCT- 7 DAS- 28 DAS)
The results are expressed as mean ± standard error (SE) of three biological replicates. Analysis of variance followed by post hoc Duncan’s Multiple Range Test (DMRT) was performed using SPSS version 26 to determine significant differences among the morphological and physio-biochemical parameters.
3. RESULTS
3.1. Physical Character Analysis
The study of AL physical parameters disclosed that the weight, length, and breadth of the ALF increased progressively from 7 DAF to its maximal value at 150 DAF (Table S1). The specific gravity of the ALF decreased from 7 DAF (1.57 ± 0.13) to 90 DAF (0.97 ± 0.01), after which it rose to 150 DAF (1.06 ± 0.02). The ALF was initially seen to be green in color till 60 DAF, after which it appears greenish yellow at 90 DAF, and then yellow throughout the 120 and 150 DAF periods (Fig. 2). Likewise, the weight of PL and PP increases from 30 DAF (35.51 ± 2.04 g, 22.41 ± 0.91 g) to its maximal value (60.10 ± 2.86 g, 119.01 ± 1.86 g) at 150 DAF. Fruit's rind thickness increases from 30 DAF (5.2 ± 0.28 mm), reaches its maximum value at 60 DAF (7 ± 0.29 mm), and then it decreases from 90 DAF (5 ± 0.16 mm) to its minimal value at 150 DAF (4 ± 0.22 mm). It was also noted that the albedo thickness increased from 30 DAF (3.57 ± 0.21 mm) to achieve its maximum value at 60 DAF (6 ± 0.22 mm) and then decreases from 90 DAF (4.27 ± 0.05 mm) to its lowest value at 150 DAF (3.57 ± 0.13 mm), whereas the flavedo thickness decreases from 30 DAF (1.63 ± 0.13 mm) to its minimum value at 150 DAF (0.43 ± 0.09 mm). In addition, LPA of the ALF increases from 30 DAF (17.92 ± 0.26 mm) to its maximal value at 150 DAF (27.98 ± 1.3 mm) (Fig. 3, Table S1).
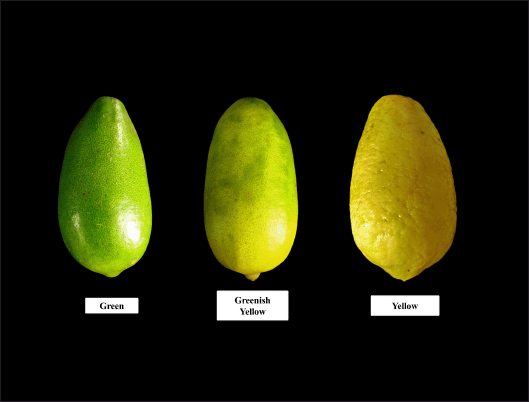 | Figure 2. Change in colour of AL at various developmental stages. [Click here to view] |
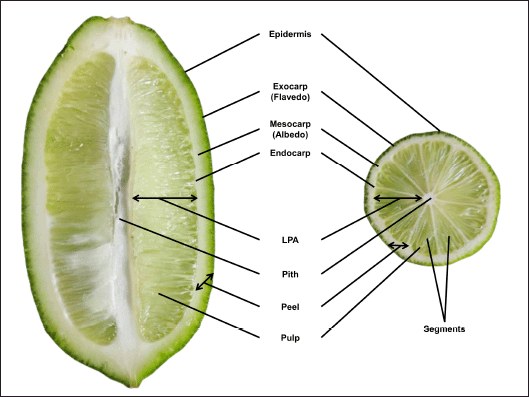 | Figure 3. Cross section of ALF. [Click here to view] |
In addition, there have been observed alterations in the physical attributes of ALF at SRT and SCT between 7th and 28th DAS (Fig. 4, Table S1). Moreover, it came into observation that the fruit weight decreases from 7 DAS (SRT = 174.28 ± 4.2 g, SCT = 178.98 ± 1.6 g) to 28 DAS (SRT = 161.92 ± 3.23 g, SCT = 176.21 ± 5 g) during both SRT and SCT. Likewise, weight of the PL and PP decreased from 7 DAS (PL – SRT = 59.28 ± 1.3 g, SCT = 59.78 ± 0.2 g and PP – SRT = 115 ± 2.86 g, SCT = 119.2 ± 1.3 g) to 28 DAS (PL – SRT = 58.78 ± 0.29 g, SCT = 59.06 ± 2.3 g and PP – SRT = 105.8 ± 1.3 g, SCT = 117.15 ± 2.6 g) at both SRT and SCT. The specific gravity also decreased from 7 DAS (SRT = 1.03 ± 0.01, SCT = 1.06 ± 0.01) to 28 DAS (SRT = 0.96 ± 0.01, SCT = 1.03 ± 0.01) at both storage conditions. It was also noted that length, breadth, pith diameter, albedo, flavedo, and rind thickness decreased gradually from 7 DAS to their lowest value at 28 DAS during SRT and SCT (Fig. 4, Table S1). Further, at SRT, the ALF appeared to be yellow in color till 15 DAS, after which, the color changed to pale yellow till 28 DAS, whereas there was no change in color (yellow) in ALF stored at SCT. In addition, the LPA of the ALF decreased from 7 DAS (SRT = 27.02 ± 0.69 mm, SCT = 27.6 ± 0.56 mm) to 28 DAS (SRT = 22.66 ± 0.53 mm, SCT = 26.37 ± 0.25 mm). However, the alterations in the physical attributes of AL were observed to be more prominent at SRT than SCT (Fig. 4, Table S1).
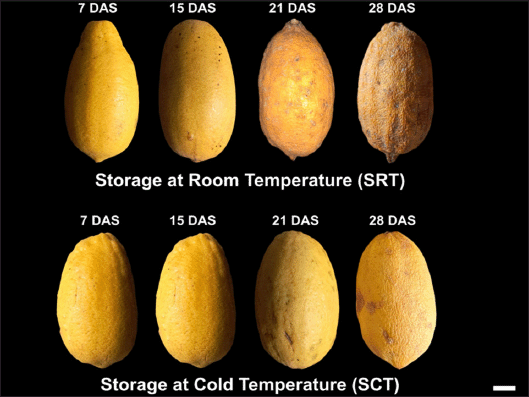 | Figure 4. Fruit morphology of ALFs at different storage temperatures (scale bar-2 cm). [Click here to view] |
3.2. Physio-Biochemical Analysis
3.2.1. pH
At DSFD, the pH was observed to be lowest at 30 DAF (2.12 ± 0.04) and then increased to its maximum at 150 DAF (3.12 ± 0.12). During post-harvest storage (PHS), the pH increases from 7 DAS (SRT = 3.45 ± 0.02, SCT = 3.31 ± 0.06) to 28 DAS (SRT = 4.46 ± 0.21, SCT = 3.97 ± 0.03). Notably, the pH increase was more pronounced at SRT compared to SCT (Table S2, Fig. 5).
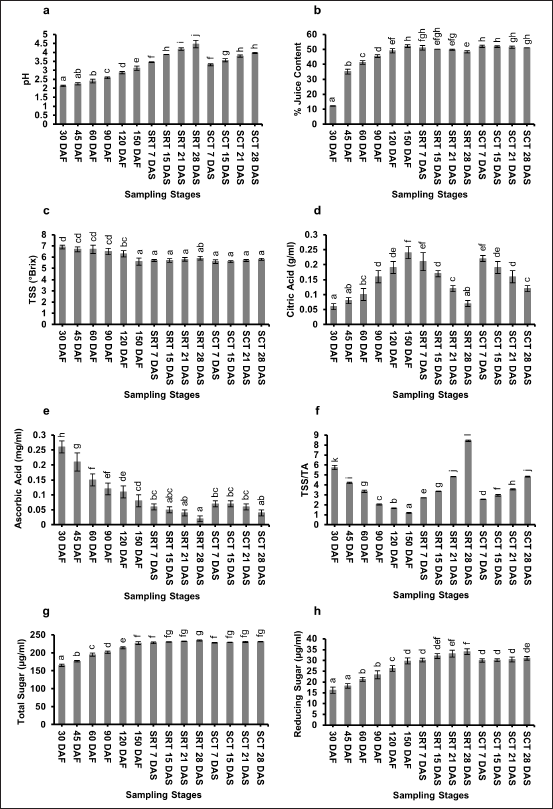 | Figure 5. Biochemical characteristics of ALF juice at DSFD (30–150 DAF) and storage (SRT- 7 DAS- 28 DAS, SCT- 7 DAS- 28 DAS) (a: pH, b: TSS, c: % JC, d: citric acid, e: ascorbic acid, f: TSS/TA, and g: TS and RS). Numerical data represent mean values (column bars) with SE of n = 3 biological replicates (three fruits total per stage/condition) represented as vertical lines on the column bars. Different letters on top of the bars represent significant differences between samples at the subset for alpha = 0.05, based on DMRT. [Click here to view] |
3.2.2. % Juice content
At DSFD, the % JC was observed to be lowest at 30 DAF (12.16% ± 0.16%) and steadily increased to its highest value at 150 DAF (52.16% ± 0.92%). During PHS, % JC decreased from 7 DAS (SRT = 51.12% ± 1.55%, SCT = 52.02% ± 0.72%) to 28 DAS (SRT = 48.42% ± 0.82%, SCT = 51.02% ± 0.04%) in both SRT and SCT. However, a decrease in % JC was more pronounced at SRT compared to SCT (Table S2, Fig. 5).
3.2.3. Total soluble solids
At DSFD, the TSS of AL juice was observed to be highest at 30 DAF (6.90 ± 0.16 °Brix) and steadily decreased to its lowest value at 150 DAF (5.60 ± 0.2 °Brix). Further, during PHS, the TSS remained unchanged from 7 DAS (SRT = 5.70 ± 0.08 °Brix, SCT = 5.60 ± 0.16 °Brix) to 15 DAS (SRT = 5.70 ± 0.16 °Brix, SCT = 5.60 ± 0.08 °Brix), and then gradually increased from 21 DAS (SRT = 5.80 ± 0.16 °Brix, SCT = 5.70 ± 0.08 °Brix) to 28 DAS (SRT = 5.90 ± 0.16 °Brix, SCT = 5.80 ± 0.08 °Brix) in both SRT and SCT. Also, the TSS rise was more at SRT compared to SCT (Table S2, Fig. 5).
3.2.4. Citric acid content (CAC)
At DSFD, the CAC in AL juice was observed to be lowest at 30 DAF (0.06 ± 0.01 g/ml), and then increases to its maximum value at 150 DAF (0.24 ± 0.02 g/ml). Again, in PHS, CAC decreased from 7 DAS (SRT = 0.21 ± 0.03 g/ml, SCT = 0.22 ± 0.01 g/ml) to 28 DAS (SRT = 0.07 ± 0.01 g/ml, SCT = 0.12 ± 0.01 g/ml), both at SRT and SCT. However, the CAC decrease was significantly pronounced at SRT compared to SCT (Table S2, Fig. 5).
3.2.5. Ascorbic acid content (AAC)
At DSFD, the AAC was highest at 30 DAF (0.26 ± 0.02 mg/ml) and steadily decreased to its lowest at 150 DAF (0.08 ± 0.02 mg/ml). In addition, during PHS, AAC decreased from 7 DAS (SRT = 0.06 ± 0.01 mg/ml, SCT = 0.07 ± 0.01 mg/ml) to 28 DAS (SRT = 0.02 ± 0.01 mg/ml, SCT = 0.04 ± 0.01 mg/ml) in both SRT and SCT. However, the AAC decrease was significantly more pronounced at SRT compared to SCT (Table S2, Fig. 5).
3.2.6. Total soluble solids/titratable acidity
At DSFD, the TSS/TA was observed to be highest at 30 DAF (5.75 ± 0.21) and subsequently decreased to its lowest at 150 DAF (1.17 ± 0.06). Further, during PHS, the TSS/TA increases from 7 DAS (SRT = 2.71 ± 0.02, SCT = 2.54 ± 0.03) to 28 DAS (SRT = 8.43 ± 0.07, SCT = 4.83 ± 0.05) in both SRT and SCT. Notably, the TSS/TA increase was significantly greater at SRT than SCT (Table S2, Fig. 5).
3.2.7. Total sugar and reducing sugar
At DSFD, the TS concentration in fruit juice of AL was lowest at 30 DAF (164.92 ± 2.98 µg/ml) and subsequently increased to its maximum value at 150 DAF (227.16 ± 4.19 µg/ml). In addition, the RS concentration was lowest at 30 DAF (16.19 ± 1.49 µg/ml), gradually increased, and reached its maximum at 150 DAF (29.76 ± 1.43 µg/ml). Further, during PHS, in both SRT and SCT, increase in TS and RS content was noted from 7 DAS (TS: SRT = 228.18 ± 2.44 µg/ml, SCT = 227.92 ± 0.98 µg/ml; RS: SRT = 30.17 ± 0.82 µg/ml, SCT = 29.98 ± 0.85 µg/ml) to 28 DAS (TS: SRT = 234.42 ± 1.44 µg/ml, SCT = 231.17 ± 0.67 µg/ml; RS: SRT = 34.08 ± 1.34 µg/ml, SCT = 30.98 ± 0.82 µg/ml). However, the increase in both the TS and RS content was noticeably greater at SRT than at SCT (Table S2, Fig. 5).
3.2.8. Carotenoid content (CC)
At DSFD, the CC was observed to be peaked at 150 DAF (2.81 ± 0.15 mg/g) after gradually increasing from its lowest point at 7 DAF (2.25 ± 0.01 mg/g). Further, during PHS, the CC increases from 7 DAS (SRT = 2.83 ± 0.02 mg/g, SCT = 2.82 ± 0.01 mg/g) to 28 DAS (SRT = 2.95 ± 0.01 mg/g, SCT = 2.92 ± 0.01 mg/g) in both SRT and SCT. However, the CC rise was significantly more at SRT compared to SCT (Table S3, Fig. 6).
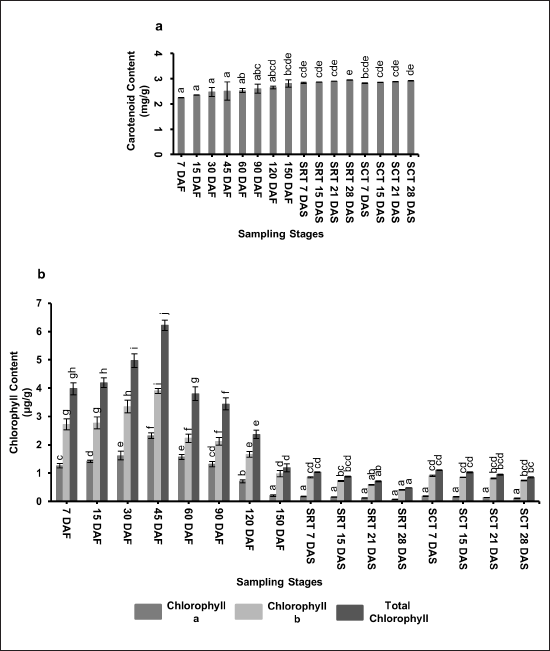 | Figure 6. Biochemical characteristics of ALF PL at DSFD (7–150 DAF) and storage (SRT- 7 DAS- 28 DAS, SCT- 7 DAS- 28 DAS) (a: CC and b: chlorophyll content). Numerical data represent mean values (column bars) with SE of n = 3 biological replicates (three fruits total per stage/condition) represented as vertical lines on the column bars. Different letters on top of the bars represent significant differences between samples at the subset for alpha = 0.05, based on DMRT. [Click here to view] |
3.2.9. Chlorophyll content
At DSFD, Chl a, Chl b, and total Chl of fruit PL of AL were observed to be highest at 7 DAF (1.26 ± 0.08, 2.72 ± 0.19, 3.98 ± 0.21 µg/g) and then rapidly decreased until it reached its lowest level at 150 DAF (0.21 ± 0.03, 0.98 ± 0.11, 1.19 ± 0.14 µg/g). Further, during PHS, Chl a, Chl b, and total Chl significantly reduced from 7 DAS (SRT = 0.18 ± 0.01, 0.85 ± 0.02, 1.03 ± 0.01; SCT = 0.19 ± 0.01, 0.91 ± 0.02, 1.10 ± 0.01 µg/g) to 28 DAS (SRT = 0.07 ± 0.01, 0.41 ± 0.01, 0.48 ± 0.01; SCT = 0.11 ± 0.01, 0.74 ± 0.01, 0.85 ± 0.02 µg/g). However, Chl a, Chl b, and total Chl decreased more rapidly at SRT compared to SCT (Table S3, Fig. 6).
3.2.10. Pectin content
At DSFD, the PC at PL was gradually increased from its lowest concentration at 7 DAF (0.42% ± 0.05%) and reached its peak value at 60 DAF (2.77% ± 0.23%), and then decreased from 90 DAF (2.44% ± 0.21%) till 150 DAF (0.89% ± 0.04%). In addition, at DSFD, the PC at PP gradually increases from 30 DAF (2.17% ± 0.17%) to reach its peak value at 60 DAF (5.26% ± 0.26%), and then decreases from 90 DAF (3.06% ± 0.23%), reaching its lowest value (1.17% ± 0.07%) at 150 DAF. Again, during the PHS, PC in both PL and PP of the ALF decreases from 7 DAS (SRT = 0.85% ± 0.01%, 1.08% ± 0.02%; SCT = 0.87% ± 0.03%, 1.12% ± 0.02%) reaching the lowest value at 28 DAS (SRT = 0.51% ± 0.02%, 0.81% ± 0.02%; SCT = 0.72% ± 0.02%, 0.95% ± 0.02%) in both SRT and SCT. However, SRT showed a greater decrease in PC than SCT (Table S4, Fig. 7).
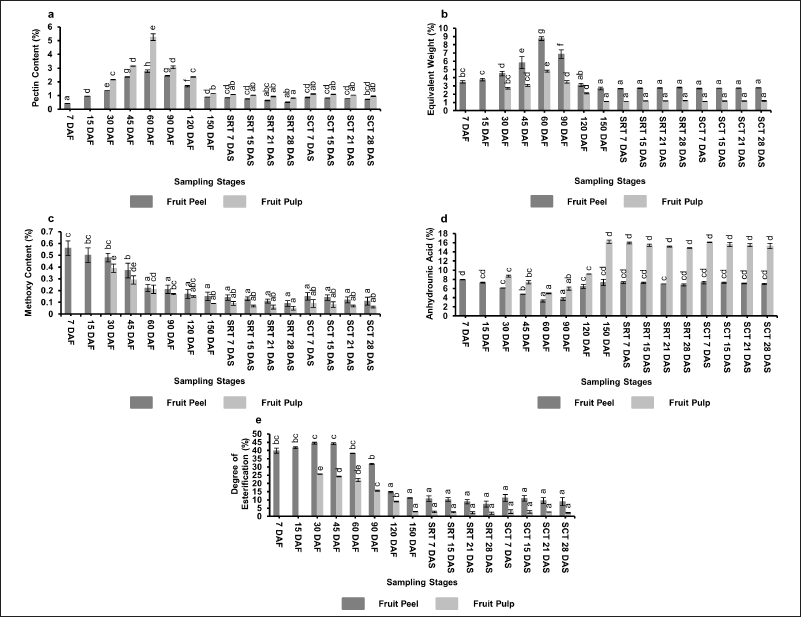 | Figure 7. Chemical characterization of pectin obtained from ALF at DSFD (7–150 DAF) and storage (SRT- 7 DAS- 28 DAS, SCT- 7 DAS- 28 DAS) (a: PC, b: EW, c: MeOC, d: AUA, and e: DE). Numerical data represent mean values (column bars) with SE of n = 3 biological replicates (three fruits total per stage/condition) represented as vertical lines on the column bars. Different letters on top of the bars represent significant differences between samples at the subset for alpha = 0.05, based on DMRT. [Click here to view] |
3.2.11. Equivalent weight
At DSFD, the EW of PL gradually rises from 7 DAF (3.49% ± 0.27%), reaches its peak value (8.73% ± 0.58%) at 60 DAF, and then decreases from 90 DAF (6.85% ± 0.54%) until it reaches its lowest value (2.69% ± 0.31%) at 150 DAF. In addition, at DSFD, the EW of PP gradually increased from 30 DAF (2.73% ± 0.35%) to reach its peak value (4.79% ± 0.73%) at 60 DAF, and then gradually decreased from 90 DAF (3.49% ± 0.42%) until it reached its lowest value (1.12% ± 0.2%) at 150 DAF. Furthermore, during PHS, EW in both PL and PP of ALF increased from 7 DAS (SRT= 2.69% ± 0.02%, 1.14% ± 0.01%; SCT = 2.71% ± 0.03%, 1.13% ± 0.02%) and reaches its peak value at 28 DAS (SRT = 2.81% ± 0.05%, 1.21% ± 0.02%; SCT = 2.77% ± 0.02%, 1.18% ± 0.04%) at both SRT and SCT. Notably, at SRT, the EW rise was more compared to SCT (Table S4, Fig. 7).
3.2.12. Methoxy content
At DSFD, the MeOC of PL was highest at 7 DAF (0.56% ± 0.14%) and then gradually decreased until it reached its lowest value (0.15% ± 0.07%) at 150 DAF. In addition, at DSFD, the MeOC of PP was observed to be highest at 30 DAF (0.39% ± 0.11%) and then gradually decreases to its lowest value (0.09% ± 0.02%) at 150 DAF. In addition, the MeOC in both PL and PP of ALF during PHS decreased from 7 DAS (SRT = 0.14% ± 0.02%, 0.09% ± 0.02%; SCT = 0.15% ± 0.03%, 0.09% ± 0.03%) and reaches its lowest value at 28 DAS (SRT = 0.09% ± 0.02%, 0.05% ± 0.02%; SCT = 0.11% ± 0.03%, 0.06% ± 0.01%) at both SRT and SCT. However, SRT showed a decrease in MeOC than at SCT (Table S4, Fig. 7).
3.2.13. Anhydrouronic acid
At DSFD, the AUA of PL was observed to be highest at 7 DAF (7.93% ± 1.16%) after which it gradually decreased to its lowest value (3.27% ± 0.67%) at 60 DAF, and then again rises from 90 DAF (3.69% ± 0.73%) till 150 DAF (7.3% ± 0.53%). In addition, at DSFD, the AUA of PP was gradually decreased from 30 DAF (8.68% ± 1.37%) to reach its lowest value (4.96% ± 0.88%) at 60 DAF, and then it gradually increased from 90 DAF (5.98% ± 0.89%), reaching its highest value (16.19% ± 2.95%) at 150 DAF. Furthermore, at storage, the AUA in both PL and PP of ALF decreases from 7 DAS (SRT = 7.28% ± 0.18%, 15.95% ± 0.2%; SCT = 7.29% ± 0.26%, 16.09% ± 0.04%) and reaches its lowest value at 28 DAS (SRT = 6.77% ± 0.25%, 14.83% ± 0.1%; SCT = 6.98% ± 0.15%, 15.27% ± 0.56%) at both SRT and SCT. However, SRT experienced a more pronounced reduction in the AUA content compared to SCT (Table S4, Fig. 7).
3.2.14. Degree of esterification
At DSFD, the DE of PL was gradually increased from 7 DAF (39.89% ± 5.01%) and reached its peak value (44.49% ± 3.3%) at 30 DAF, and then decreased from 45 DAF (44.11% ± 4.83%) until it reached its lowest value (11.15% ± 5.81%) at 150 DAF. In addition, DE of ALF PP was highest (25.67% ± 3.23%) at 30 DAF and then from 60 DAF (24.18% ± 2.92%) DE rapidly decreased until it reached its lowest value (2.88% ± 0.74%) at 150 DAF. Furthermore, during PHS, the DE of PC in both PL and PP of ALF decreases from 7 DAS (SRT = 10.79% ± 1.63%, 2.72% ± 0.54%; SCT = 11.14% ± 2.11%, 2.86% ± 1.16%) and reaches its lowest value at 28 DAS (SRT = 7.48% ± 1.78%, 1.92% ± 0.64%; SCT = 8.9% ± 2.47%, 2.22% ± 0.22%) at both SRT and SCT. Notably, SRT exhibited a greater decrease in DE compared to SCT (Table S4, Fig. 7).
3.3. Soil Nutrient Estimation
The assessment of soil nutrients from the AL collection site during DSFD indicated minimal variation across different collection phases. The soil was found to be slightly alkaline (7.5) and rich in several significant micro and macro nutrients. The findings from the current study demonstrated that the soil contains significant amounts of iron (> 6 ppm) and copper (0.5–2 ppm), whereas it contains comparably small amounts of zinc (0–0.5 ppm), boron (0.1–1 ppm), manganese (0–2 ppm), and molybdenum (0–0.1 ppm). The soil also contains a considerable amount of organic carbon (0.300%–0.500%), phosphate (56–73 kg/ha), and potassium (112–280 kg/ha), while ammoniacal nitrogen (15 kg/ha) and nitrate nitrogen (4 kg/ha) are present in very small proportions (Table S5).
4. DISCUSSION
AL is considered a health-protective fruit due to its nutritious content and the presence of a variety of bioactive chemicals [16]. The physio-biochemical contents, however, fluctuate significantly during DSFD [17]. It was observed in the current study that the size and weight of ALF increase as the fruit grows, attaining their maximum value at 150 DAF, which corroborated the findings of Mukhim et al. [17], and Shahida et al. [18]. The rapid cell differentiation is likely to have resulted in faster rates of increase in size and weight during the early stages of fruit development [19]. Again, during PHS, the size decreased from 7 DAS to 28 DAS (Table S1), and the decrease was slighter at SCT than SRT, which showed similarity with the results obtained by Kashyap et al. [20]. This indicates that the fruit size and weight loss can be significantly influenced by storage temperature. Further, it was noted that the LPA increased and peaked at 150 DAF. However, during storage, the LPA was greatly reduced, whereas SRT showed a higher reduction than SCT (Table S1). LPA may have increased from 7 to 150 DAF due to its dependence on the size of ALF, which influenced it to increase as the fruit size grew larger, but the decrease in LPA during storage might be due to the reduction in fruit size, which was influenced by storage temperature [17,20]. Further, the increase in fruit weight during the DSFD is primarily due to development and maturation, such as the buildup of water content, sugars, and other solutes at DSFD [21], but the decrease in fruit weight during storage might be due to the loss of water. Further, the highest specific gravity was measured at 7 DAF, and the value decreased till 90 DAF, after which it slightly increased at 150 DAF. However, the specific gravity of ALF decreases gradually from 7 to 28 DAS at both SRT and SCT. The decline in specific gravity during storage was due to the reduction in fruit size and weight, which might have resulted from loss of water. The results from specific gravity are similar to those reported by Mukhim et al. [17] but contrary to those found by Shahida et al. [18]. The fruit's weight and size have the largest impact on specific gravity change, which might be the reason behind the results obtained in the study [22].
The AL fruit's color changes from green to yellow at 90 DAF, and during storage, the fruit color changes from yellow to pale yellow at 21 DAS at SRT. The color change might be due to the Chl breakdown and carotenoid buildup in the fruit skin [23]. On the other hand, the PP to PL ratio rises from 30 DAF and reaches 150 DAF. This could be due to the fast cell differentiation and the accumulation of water, sugar, and other solutes in the juice sacs of PP [24]. However, the PP to PL ratio declines during storage at both SRT and SCT, but the reduction in the PP to PL ratio was reported to be slower at SCT than at SRT. The results of the current investigation corroborated the findings of Citrus grandis L. Osbeck [25] and Citrus unshiu [26]. Several studies reported that the rind thickness grows at maturity but reduces as the fruit ripens, and during storage [27]. Similarly, it was noted that the fruit's rind thickens and starts increasing from 30 DAF, reaches a maximum value at 60 DAF, and then subsequently decreases from 90 DAF. In addition, the rind thickness decreases during storage at both SRT and SCT; however, the decrease in rind thickness was reported to be slower at SCT than at SRT. In addition, as the fruits mature, flavedo size increases, but albedo size significantly decreases after 60 DAF. During fruit ripening, the albedo often thickens until the fruit reaches maturity, whereas the flavedo progressively thickens until the fruit abscises from the tree, which may be the reason for the current experimental results [29,30]. On the other hand, during storage, both the flavedo and albedo undergo a size reduction. This decrease occurs in the fruit irrespective of storage conditions. However, the decline in both flavedo and albedo is slower at SCT compared to SRT, which can be explained by the high rate of fruit respiration and water loss during storage [31].
It was observed that the % JC increased progressively from 30 DAF and reached its peak at 150 DAF, which is supported by the findings of Mukhim et al. [17]. The increase in JC might be due to the accumulation of water and solutes in the juice vesicles [21]. Also, fruit ages lead to an increase in JC, which might be the result of juice formation and accumulation inside the juice sacs [32]. On the other hand, during storage, the % JC was observed to decrease in both SRT and SCT due to the loss of water and solutes in the juice vesicle [17]. Again, the TSS/TA content during the DSFD steadily decreases from 30 DAF and reaches its lowest value at 150 DAF. However, during the storage, the TSS/TA rose from 7 DAS to 28 DAS at both SRT and SCT. The rapid reduction in TSS and substantially greater rates of acid buildup might be the cause of the decline in the TSS/TA ratio during the DSFD, but during storage, an opposite trend was observed, leading to an increase in the TSS/TA ratio [17,20]. Nevertheless, AAC also gradually declines from 30 to 150 DAF, where it hits its lowest level. Similarly, during storage, at both SRT and SCT, the AAC gradually decreased from 7 DAS and reached its lowest value at 28 DAS. The use of ascorbic acid in certain metabolic processes might be the cause of the ascorbic acid's decrease during the maturation process [33].
During the study, we also observed that there is an increase in pH with the maturity of fruits. Furthermore, during storage, the pH levels showed an upward trend, indicating a shift toward alkalinity. However, it was noteworthy that the inclination of pH at SRT was more pronounced compared to SCT. In addition, it was also revealed that the TS and RS rise during the fruit ripening and storage, which might be a key element affecting the pH of ALF [34]. The result was supported by the findings on Citrus sinensis L. Osbeck [35], Citrus aurantifolia Swingle [36], Citrus reticulata Blanco [20], and other plants. Again, during the current investigation, we observed that the citric acid concentration of ALF increases as the fruit ripens, which might be due to the synthesis by enzymatic activity in juice vesicles during fruit development [17]. It was earlier reported that ALF could remain on the plant for an extended period of time after they were fully ripe, which may be due to an increase in citric acid concentration [5,36]. In addition, during the current experiment, a decline in the citric acid concentration was observed as the storage period progressed. However, a noteworthy finding was that the decrease in CAC was observed to be slower at SCT compared to SRT. The decline in CAC could be due to the breakdown of citric acid in the Krebs' cycle, which occurs during the aerobic respiration process [20].
In the present study, we investigated the changes in Chl a, Chl b, and total Chl content during fruit growth stages. In addition, we observed the change in Chl levels during both SRT and SCT, which has not been reported yet. It was revealed that the concentration of Chl a, Chl b, and total Chl decreases while the concentration of carotenoid rises as the fruit ripens and during storage [37,38]. This might be due to the lycopene buildup and the transformation of Chl to carotenoid during fruit ripening [38–40].
Pectin in Citrus is an important ingredient used in different food processing industries [41]. During the current investigation, we noticed that PL and PP of ALF contained a significant amount of pectin, with PP having greater PC than PL throughout the fruit development stages. Again, it was observed that the PC in PL and PP of ALF gradually increased and reached its peak at 60 DAF and then sharply decreased. The activity of several pectin-degrading enzymes, including lyase, pectin methylesterase, polygalacturonase, rhamnogalacturonase, etc., may be the cause of the decrease in PC [42]. In addition, at SRT and SCT, we noticed a consistent decrease in pectin levels as the storage duration advanced. However, the reduction in PC was notably more pronounced at SRT compared to SCT. The degradation of pectin during storage might be due to the activity of pectinases, pectin methylesterase, etc., which act during the breakdown of the pectin molecules in the cell wall of fruits [43–45]. Factors like temperature and an increase in the activity of ethylene during storage further accelerate this enzyme activity, which might be the reason for the reduction in PC in ALF [46,47]. Similar results were also observed in C. limon L. Osbeck [48] and Prunus persica L. Batsch [49].
EW of PC in PL and PP of ALF gradually increased and reached its peak at 60 DAF, after which it rapidly decreased till 150 DAF. However, during storage, it was observed that the EW of PL and PP gradually increased from 7 DAS till 28 DAS at both SRT and SCT. Again, on measuring the MeOC, we observed that the MeOC was maximum at the initial stage, which gradually declined to its lowest value at 150 DAF. Similarly, throughout the storage period, MeOC gradually declined from 7 to 28 DAS, with the maximum decrease observed in SRT compared to SCT. In addition, AUA (for the study of purity of the PC) was steadily decreasing from the initial stage, reaching its lowest value in 60 DAF, then continuing to increase again from 90 DAF. This suggests that the pectin in AL attained its highest purity during the fruit's ripening and early stages of fruit development. On the other hand, during storage, the AUA content gradually decreased from 7 to 28 DAS in both PL and PP of ALF, with the most significant decrease at SRT compared to SCT. The pectinase activity can lead to the depolymerization of pectin, reducing overall purity [50]. Furthermore, while studying the pectin's level of esterification to determine the concentration of methylesters, which is either high-methoxy pectin or low-methoxy pectin depending on the extent of esterification, it was revealed that pectin found in both AL-PL and AL-PP was low-methoxy pectin (<50%) [51]. Similar findings have been reported in Citrus maxima Burm Merr, Citrus jambhiri Lush, Citrus suduchi, Citrus hystrix DC, Citrus limetta Risso, C. sinensis L. Osbeck, C. limon L. Osbeck [52,53], and others.
Significant physio-biochemical variations were observed in both PL and PP of the ALF during the DSFD and storage. It was also observed that the samples at SRT exhibited a significant decline in physio-biochemical parameters compared to samples at SCT, which is a critical factor in maintaining the desired physio-biochemical parameters for various applications [54]. Since each food and pharmaceutical industry has different needs, these industries look into different physio-biochemical factors for the selection of quality fruits for different products to be produced [55]. These industries, therefore, might employ the appropriate fruit stage of ALF as a source of raw material for their products. An estimation of the nutritional value of ALF in various stages is expected to promote such endeavours [54]. Therefore, different harvesting and storage times for ALF may be required based on their industry product development requirements.
The quantity of both macronutrients and micronutrients in the soil is an important aspect that influences a Citrus natural growth and development and could alter not just fruit yield but also the amount of nutrients in fruits [28,56–59]. Several studies have reported that the phosphate, potassium, and nitrogen levels in the soil can influence the yield and size of Citrus fruits [60]. In the current study, soil pH at the sample collection site was about 7.5, the level of organic carbon was between 0.30% and 0.500%, and phosphate and potassium concentrations were found to be 56 –73 and 112–280 kg/ha, respectively, which is considered to be ideal for the normal growth of Citrus plants [61,62]. It was also noticed that nitrogen present (ammoniacal nitrogen and nitrate nitrogen) in the soil is about 19 kg/ha, which is an optimal value for the growth and development of various plant species [63]. Further, it was also observed that the micronutrients present at the sample collection site, which include copper (0.5–2 ppm), zinc (0–0.5 ppm), boron (0.1–1 ppm), manganese (0–2 ppm), iron (> 6 ppm), and molybdenum (0–0.1 ppm), are in the ideal range for Citrus growth [61,64]. Similar observations were also noticed in C. sinensis L. Osbeck [59], Citrus nobilis Lour [65], C. reticulata Blanco [65], C. aurantifolia Swingle [66], others, suggesting that normal plant growth and the development of fruit quality and yield are significantly influenced by soil nutrient status [59,65,66]. A relationship between soil nutrient characteristics and fruit quality has also been reported in Xinjiang jujube [28]. Although these soil parameters give a significant understanding of the soil condition and its influence on the morphological and physio-biochemical variation of AL, the values obtained were interpreted as indicative rather than definitive measures of absolute soil nutrient concentrations, as the results provided semi-quantitative estimates rather than highly precise analytical measurements. The findings of this study open the door for advanced and more precise research and their influence on Citrus morphological and physio-biochemical variation at different stages of fruit growth and development.
5. CONCLUSION
The current study was carried out to gain a comprehensive understanding of physical and physio-biochemical changes during DSFD and storage conditions. The study emphasizes how the key physio-biochemical characteristics of AL change during fruit development and during various conditions of storage. Most quality-related parameters, including pH, JC, sugars, citric acid, and carotenoids, reached their peak at full maturity (150 DAF); however, several other important biochemical constituents attained their maximum levels at DSFD. In addition, during storage, morphological and physio-biochemical traits exhibited greater stability under SCT compared to SRT. These findings provide valuable insights for optimizing harvest timing, storage strategies, and industrial utilization, particularly in food processing and pharmaceutical applications. This cognizance of the dynamic morphological and physio-biochemical transformations within fruit PL and PP throughout their development and storage is a cornerstone for elevating agricultural practices, enhancing the quality and safety of food products, and meeting the standards of diverse industries, including pharmaceuticals. This understanding would help stakeholders to make informed decisions and ultimately ensure that consumers have access to fresh, high-quality produce while also driving advancements in the field of agriculture and food science.
6. ACKNOWLEDGMENT
The authors are indebted to Gauhati University for providing the technical facility. The authors also acknowledge the Department of Biotechnology, Government of India, under the Task Force scheme for providing the financial aid vide sanction number BT/PR21144/BPA/118/203/2016.
7. AUTHOR CONTRIBUTIONS
All authors made substantial contributions to conception and design, acquisition of data, or analysis and interpretation of data; took part in drafting the article or revising it critically for important intellectual content; agreed to submit to the current journal; gave final approval of the version to be published; and agreed to be accountable for all aspects of the work. All the authors are eligible to be authors as per the International Committee of Medical Journal Editors (ICMJE) requirements/guidelines. Original draft preparation, investigation, acquisition of data, analysis, and interpretation of data were performed by Raja Ahmed and Suraiya Akhtar. Raja Ahmed and Suraiya Akhtar contributed equally to this work and share first authorship. Writing, analysis, interpretation of data, and substantial revision of the article were done by Raja Ahmed and Suraiya Akhtar. The article was reviewed by Ankur Das and Khaleda Begum. Availability of experimental materials was done by Dikshita Saikia and Sarat Saikia. The conception, study design, supervision, critical review, and article revision were done by Sofia Banu. All authors read and approved the final manuscript. The authors also declare no conflict of interest.
8. FUNDING
This work was supported by the Department of Biotechnology, Government of India, under Task Force (sanction number BT/PR21144/BPA/118/203/2016).
9. CONFLICTS OF INTEREST
The authors report no financial or any other conflicts of interest in this work.
10. ETHICAL APPROVALS
This study does not involve experiments on animals or human subjects.
11. DATA AVAILABILITY
All data are available from the authors and will be provided upon request. Data are contained within the article and are attached as Supplementary Materials.
12. PUBLISHER’S NOTE
All claims expressed in this article are solely those of the authors and do not necessarily represent those of the publishers, the editors, or the reviewers. This journal remains neutral about jurisdictional claims in published institutional affiliation.
13. USE OF ARTIFICIAL INTELLIGENCE (AI)-ASSISTED TECHNOLOGY
The authors declare that they have not used AI-tools for writing and editing of the manuscript, and no images were manipulated using AI.
14. SUPPLEMENTARY MATERIAL
The supplementary material can be accessed at the journal’s website: https://jabonline.in/admin/php/uploadss/1507_pdf.pdf
REFERENCES
1. Pavia JL. 31 types of lemons and what makes them unique. Tasting Table. 2023. Available via https://www.tastingtable.com/906950/types-of-lemons-and-what-makes-them-unique/ (Accessed 6 June 2024)
2. Lakhan Y. 7 popular lemon varieties found in India. Slurrp. 2022. Available via https://www.slurrp.com/article/7-popular-lemon-varieties-found-in-india-1656079726793 (Accessed 7 February 2024)
3. Ahmed R, Akhtar S, Das A, Begum K, Kashyap K, Banu S. Delineating the degree of genetic divergence within Assam lemon (Citrus limon ‘Assam lemon’) accessions in Assam, India. Genet Resour Crop Evol. 2023;70(8):2785–2799.
4. Barua BC, Bharadwaj S. Assam lemon – a prospective NPD initiative aimed at global market positioning. Int J Res 2017;4(14):727–34.
5. Crs-Na-Dihing Nemu Tenga Unnayan Samity (2019). G.I. application number – 609. Geogr Indic J 2019;123:13–21.
6. Karelia G, Rao Y. Assam’s ‘accidental’ seedless lemon variety doubles farmer profits in UK. The better India. 2021. Available via https://www.thebetterindia.com/260719/assam-village-exports-kaji-nemu-lemon-uk-profits-gi/#:~:text=Assam's%20'Accidental'%20Seedless%20Lemon%20Variety%20Doubles%20Farmer%20Profits%20in%20UK,-By%20Gopi%20Karelia&text=Grown%20in%20Panbari%20village%20of,Sounds%20Interesting%3F (Accessed 2 August 2024)
7. Thakur S. 2010. World’s first experimental plantation of grafted Assam lemon raised at Kahikuchi. Assam Tribune. 2010. https://assamtribune.com/worlds-first-experimental-plantation-of-grafted-assam-lemon-raised-at-kahikuchi#:~:text=Using%20the%20seeds%20of%20China,others%20and%20had%20seedless%20fruit (Accessed 1 August 2024)
8. Lv X, Zhao S, Ning Z, Zeng H, Shu Y, Tao O, et al. Citrus fruits as a treasure trove of active natural metabolites that potentially provide benefits for human health. Chem Cent J. 2015;9:68; CrossRef
9. Albornoz PL, Interdonato R, Hammann A, Rosa M, Prado FE, Rapisarda VA, et al. Lemon maturation causes anatomical and biochemical changes at the flavedo tissue level. Botany 2022;100(4):347–57.
10. Weibel FP, Alfoldi T. Improving the quality and shelf life of fruit from organic production systems. In: Cooper J, Niggli U, Leifert C (eds.). Handbook of organic food safety and quality, Woodhead Publishing, pp 330–52, 2007; CrossRef
11. Maldonado-Celis ME, Yahia EM, Bedoya R, Landázuri P, Loango N, Aguillón J, et al. Chemical composition of Mango (Mangifera indica L.) fruit: nutritional and phytochemical compounds. Front Plant Sci. 2019;10:1073; CrossRef
12. Zainalabidin FA, Sagrin MS, Azmi WNW, Ghazali AS. Optimum postharvest handling-effect of temperature on quality and shelf life of tropical fruits and vegetables. J Trop Resour Sustain Sci 2019;7:23–30; CrossRef
13. Hoffmann TG, De Souza CK, Sonawane AD, Praeger U, Büchele F, Neuwald DA, et al. Challenges and future perspectives in postharvest cold storage: technological review on sustainable and efficient cold storage of fresh produce. Food Res Int 2025;221:117406; CrossRef
14. Afriyie E, Zurek M, Asem FE, Okpattah B, Ahiakpa JK, Zhu YG. Consumer food storage practices and methods at the household-level: a community study in Ghana. Front Sustain Food Syst 2023;7:1194321; CrossRef
15. Akhtar S, Ahmed R, Begum K, Das A, Saikia S, Laskar RA, et al. Evaluation of morphological traits, biochemical parameters and seeding availability pattern among Citrus limon ‘Assam lemon’ accessions across Assam. Sci Rep 2024;14:3886; CrossRef
16. Gogoi M. Assam lemon: a magical fruit. E-Zine Bio Sci 2021;19:1–4.
17. Mukhim C, Nath A, Deka B, Swer TL. Changes in physicochemical properties of Assam lemon (Citrus limon burm.) At different stages of fruit Growth and development. Bioscan 2015;10(2):535–7.
18. Shahida C, Manisha K, Mridul D. Physicochemical changes in Assam Lemon (Citrus limon Burm.) during fruit development and maturation. Int J Env Clim Change 2022;12(6):90–4; CrossRef
19. Padmanabhan P, Cheema A, Paliyath G. Solanaceous fruits including tomato, eggplant, and peppers. In: Caballero B, Finglas PM, Toldra F (eds.). Encyclopedia of food and health. 3rd edition, Cambridge, UK: Academic Press; pp 24–32, 2016; CrossRef
20. Kashyap K, Kashyap D, Nitin M, Ramchiary N, Banu S. Characterizing the nutrient composition, physiological maturity, and effect of cold storage in Khasi Mandarin (Citrus reticulata Blanco). Int J Fruit Sci 2020;20(3):521–40; CrossRef
21. Hou X, Zhang W, Du T, Kang S, Davies WJ. Responses of water accumulation and solute metabolism in tomato fruit to water scarcity and implications for main fruit quality variables. J Exp Bot 2020;71(4):1249–64; CrossRef
22. Chandra Naithani D, Rawat JMS, Singh B, Khanduri VP, Riyal MK. Determination of physicochemical properties of Aonla (Emblica officinalis Gaerth) fruits among different populations in Garhwal Himalaya. Int J Fruit Sci 2020;20(S3):S1579–89; CrossRef
23. Kapoor L, Simkin AJ, George Priya Doss C, Siva R. Fruit ripening: dynamics and integrated analysis of carotenoids and anthocyanins. BMC Plant Biol 2022;22:27; CrossRef
24. Aquino CF, Salomão LCC, Cecon PR, Siqueira DLD, Ribeiro SMR. Physical, chemical and morphological characteristics of banana cultivars depending on maturation stages. Rev Caatinga 2017;30(1):87–96; CrossRef
25. Gupta AK, Dhua S, Sahu PP, Abate G, Mishra P, Mastinu A. Variation in phytochemical, antioxidant and volatile composition of Pomelo fruit (Citrus grandis (L.) Osbeck) during seasonal growth and development. Plants 2021;10(9):1941; CrossRef
26. Kim SS, Kim HJ, Park KJ, Kang SB, Park Y, Han SG, et al. Metabolomic profiling of Citrus unshiu during different stages of fruit development. Plants 2022;11(7):967; CrossRef
27. Singh A, Swami S, Panwar NR, Kumar M, Shukla AK, Rouphael Y, et al. Development changes in the physicochemical composition and mineral profile of Red-Fleshed Dragon fruit grown under semi-arid conditions. Agron 2022;12(2):355; CrossRef
28. Wang C, He W, Kang L, Yu S, Wu A, Wu W. Two-dimensional fruit quality factors and soil nutrients reveals more favorable topographic plantation of Xinjiang jujubes in China. PLoS One 2019;14(10):e0222567; CrossRef
29. Sadka A, Shlizerman L, Kamara I, Blumwald E. Primary metabolism in Citrus fruit as affected by its unique structure. Front Plant Sci 2019;10:1–4; CrossRef
30. Hall CB, Augustine JJ, Lazarte JE. Pericarp thickness of ripened Tomato fruit related to maturity at harvest. Hort Sci 1979;14(4):541–2.
31. Mikasari W, Calista I, Mussadad D, Fauzi E, Megawati N, Puspitasari M, et al. Physical quality change in orange fruit (RGL variety): effects of different temperatures in storage. In IOP Conference Series Earth and Environmental Science, IOP Publishing Ltd, Purwokerto, Indonesia, 2021. Vol. 653, p 012142; CrossRef
32. Angami T, Kalita H, Baruah S, Ronya T, Bam B, Shukla KK. Dynamics of physico-biochemical changes in passion fruit varieties across maturity. Int J Chem Stud 2017;5(6):162–5.
33. Padayatty SJ, Levine M. Vitamin C physiology: the known and the unknown and Goldilocks. Oral Dis 2016;22(6):463–93; CrossRef
34. Bigard A, Romieu C, Sire Y, Veyret M, Ojéda H, Torregrosa L. The kinetics of grape ripening revisited through berry density sorting. Oeno One 2019;4:709–24; CrossRef
35. Strazzer P, Spelt CE, Li S, Bliek M, Federici CT, Roose ML, et al. Hyperacidification of Citrus fruits by a vacuolar proton-pumping P-ATPase complex. Nat Commun 2019;10:1; CrossRef
36. Samaradiwakara SD, Champa WAH, Eeswara JP. Harvest maturity affects postharvest quality of lime fruits (Citrus aurantifolia Swingle). Trop Agric Res 2019;30(4):125–31; CrossRef
37. Zhang JY, Pan DL, Jia ZH, Wang T, Wang G, Guo ZR. Chlorophyll, Carotenoid and Vitamin C metabolism regulation in Actinidia chinensis 'Hongyang' outer pericarp during fruit development. PLoS One 2018;13(3):e0194835; CrossRef
38. Conesa A, Manera FC, Brotons JM, Fernandez-Zapata JC, Simón I, Simón-Grao S, et al. Changes in the content of chlorophylls and carotenoids in the rind of Fino 49 lemons during maturation and their relationship with parameters from the CIELAB color space. Sci Hortic 2019;243:252–60; CrossRef
39. Patil SR, Sonkamble AM, Debaje PP. Fruit development and maturity of mrig bahar Nagpur mandarin fruits. Asian J Hort 2016;11(1):151–3; CrossRef
40. Su L, Diretto G, Purgatto E, Danoun S, Zouine M, Li Z, et al. Carotenoid accumulation during tomato fruit ripening is modulated by the auxin-ethylene balance. BMC Plant Biol 2015;15:114; CrossRef
41. Freitas CMP, Coimbra JSR, Souza VGL, Sousa RCS. Structure and applications of pectin in food, biomedical, and pharmaceutical industry: a review. Coatings 2021;11(8):922; CrossRef
42. UKEssays. Role of pectin enzymes in fruit ripening process. 2021. Available via https://www.ukessays.com/essays/sciences/role-pectic-enzymes-fruit-ripening-6817.php (Accessed 29 August 2024)
43. Bajpai P. Industrial applications of thermophilic/hyperthermophilic enzymes. In: Bajpai P (ed.). Developments and applications of enzymes from thermophilic microorganisms, Elsevier, pp 105–284, 2023; CrossRef
44. Gebregziabher AA, Supriyadi S, Indarti S, Setyowati L. Texture profile and pectinase activity in tomato fruit (Solanum lycopersicum, Servo F1) at different maturity stages and storage temperatures. Planta Tropika 2021;9(1):20–34; CrossRef
45. Meena B, Sowmeya VG, Praveen AB, Swetha A, Chandra DNS, Kavitha M. Pectin degradation in fruit juices by pectinase from Meyerozyma sp. VITPCT75 isolated from Phyllanthus emblica. J Pure Appl Microbial 2021;15(2):926–35; CrossRef
46. Xu M, Zhou W, Geng W, Zhao S, Pan Y, Fan G, et al. Transcriptome analysis insight into ethylene metabolism and pectinase activity of apricot (Prunus armeniaca L.) development and ripening. Sci Rep 2021;11:13569; CrossRef
47. Biz A, Farias FC, Motter FA, De Paula DH, Richard P, Krieger N, et al. Pectinase activity determination: an early deceleration in the release of reducing sugars throws a spanner in the works!. PLoS One 2014;9(10):e109529; CrossRef
48. Frempong KEB, Chen Y, Liang L, Lin X. Effect of calcium chloride and 1-methylcyclopropene combined treatment on pectin degradation and textural changes of Eureka lemon during postharvest storage. Curr Res Food Sci 2022;5:1412–21; CrossRef
49. Bakshi P, Masoodi FA. Enzymological changes in peach cv. Flordasun during storage. Indian J Hort 2010;67(2):238–42.
50. Singh Jadaun J. Pectinase: a useful tool in fruit processing industries. Nutri Food Sci Int J 2018;5(5):555673; CrossRef
51. Vanitha T, Khan M. Role of pectin in food processing and food packaging. In: Masuelli MA (ed.). Pectins. 1st edition. London, UK: IntechOpen, pp 1–21, 2019; CrossRef
52. Baraiya K, Yadav VK, Choudhary N, Ali D, Raiyani D, Chowdhary VA, et al. A comparative analysis of the physico-chemical properties of Pectin isolated from the peels of seven different Citrus fruits. Gels 2023;9(11):908; CrossRef
53. Ahmed S, Sikder MBH. Extraction, characterization and application of three varieties of Citrus limon L. pectin in jelly product. Food Appl Biosci J 2019;7(1):31–50.
54. Kumari S, Dhingra D. Post-harvest management of fruits in India: a review. J Agric Engg 2024;61(2):181–201; CrossRef
55. Quaggio JA, Mattos D Jr, Cantarella H, Almeida ELE, Cardoso SAB. Lemon yield and fruit quality affected by NPK fertilization. Sci Hortic. 2002;96(1–4):151–162. CrossRef
56. Kumari B, Kumar L, Soni AK. Effect of micro-nutrients on growth, yield and quality of lemon (Citrus limon L.) in rainy season. Int Pharma Innov J 2022;11(2):1958–62.
57. Rahman R, Sofi JA, Javeed I, Malik TH, Nisar S. Role of micronutrients in crop production. Int J Curr Microbiol App Sci 2020;11:2265–87.
58. Shrivastav P, Prasad M, Singh TB, Yadav A, Goyal D, Ali A, et al. Role of nutrients in plant growth and development. In: Naeem M, Ansari AA, Gill SS (eds.). Contaminants in agriculture, Springer, pp 43–59, 2020; CrossRef
59. Sikarwar PS, Tomar KS. Effect of micronutrients on growth, yield and quality parameters of sweet orange (Citrus sinensis L.) cv. Mosambi. Int J Microbiol App Sci 2019;8(11):2524–30.
60. Uthman A, Garba Y. Citrus mineral nutrition and health benefits: a review. In: Gonzatto MP, Santos JS (eds.). Citrus research: horticulture and human health aspects, London, UK: IntechOpen, pp 31–7, 2023; CrossRef
61. Srivastava AK, Kohli RR. Soil suitability criteria for Citrus: an appraisal. Agri Rev 1997;18(3):139–46.
62. Chapman HD. The evaluation and management of Citrus soil. Indian J Hort 1961;18:251–76.
63. International Rice Research Institute. Nutrient management. Knowledgebank. 2007. Available via http://www.knowledgebank.irri.org/ericeproduction/IV.3_Nutrient_calculator.htm (Accessed 6 June 2024)
64. Srivastava AK, Singh S. Soil analysis based diagnostic norms for Indian Citrus cultivar. Commun Soil Sci Plant Anal 2007;33(11-12):1689–706; CrossRef
65. Devy NF, Dwiastuti ME, Hardiyanto. Effect of different soil fertility on growth and development of two Citrus cultivars under two locations. In IOP Conference Series: Earth and Environmental Science, IOP Conf Ser Earth Environ Sci. 2022;985(1):012033. CrossRef
66. Bastakoti S, Nepal S, Sharma D, Shrestha AK. Effect of foliar application of micronutrients on growth, fruit retention and yield parameters of acid lime (Citrus aurantifolia Swingle). Cogent Food Agric 2022;8:2112421; CrossRef